Breeders have developed a range of degu coat colours, some quite different from the natural agouti coat. Selecting a colour requires more than producing an unusual appearance: health, behaviour and genetic diversity must take priority.
Like Octodons.fr, World of Degus encourages adoption rather than purchasing animals from pet shops or breeders. Breeding standards can help organise selection and health monitoring, but do not by themselves prevent inherited disease or physical abnormalities. Anyone planning to breed must also check the rules that apply locally; in France, the requirements depend on the activity and applicable thresholds, rather than a certificate being automatically required for every litter.
Introduction to coat-colour genetics
Two main pigments contribute to mammalian hair colour: eumelanin, which produces brown-to-black tones, and pheomelanin, which produces yellow-to-red tones. Their amounts, distribution and deposition within the hair help determine the visible coat. Pigment production and transport are controlled by several genes and cellular processes. 1
An allele is a version of a gene. At a given locus, an animal is homozygous when it has two identical alleles and heterozygous when its two alleles differ. These terms describe the pair of alleles carried by an individual; they are not two different kinds of gene. An allele does not necessarily correspond to a single, independent colour.
The genotype is the genetic constitution under discussion; the phenotype comprises observable characteristics. In a simple dominant–recessive model, one copy of a dominant allele can be sufficient for the corresponding trait to appear, whereas a recessive trait generally requires two copies. Real pigmentation can involve interactions among genes, so a phenotype cannot always reveal the complete genotype.
In codominance, both alleles are expressed distinctly. This is different from assuming that two dominant colours automatically blend into an intermediate shade. 7 A locus is a position in the genome. Functional interaction between genes is also different from genetic linkage, which concerns their tendency to be inherited together.
Laboratory inbred strains are developed over many generations to increase genetic uniformity. Congenic strains are used to study a particular genetic region against a largely shared background. They can reduce some sources of variation, but do not guarantee identical animals or eliminate all experimental bias. 2 This research practice is not a recommendation to mate related pet degus to obtain a desired colour.
A simple inheritance example
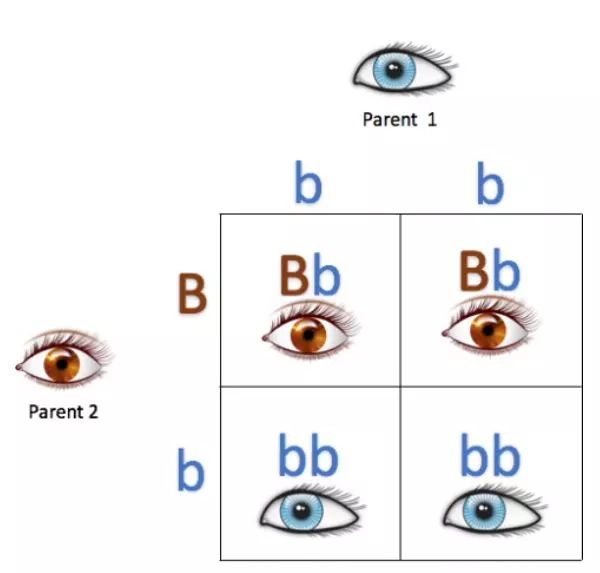
Consider an illustrative trait with a dominant allele B and a recessive allele b. A cross between bb and Bb gives each offspring a 50% probability of being bb and a 50% probability of being Bb. A cross between bb and BB gives only Bb offspring under this model. These are probabilities for each birth, not a guarantee that a small litter will contain equal numbers.
The original example used brown and blue human eyes. Human eye colour is influenced by multiple genes, so this one-locus model must not be presented as an exact prediction of a child’s eye colour. 6
The colour codes used by degu breeders
Degutopia and breeder resources use a six-locus notation to describe coat colours. This is a useful account of breeder observations and working models, but the cited pages do not establish that all six causal variants have been molecularly identified and validated in Octodon degus. The codes below retain that convention and should be read in that context. 4 5
- A — Agouti: used for banded hairs (A) and non-agouti coats (aa).
- B — Brown: used to describe brown/chocolate variation in eumelanin. It is misleading to define bb simply as the presence of pheomelanin instead of eumelanin.
- C — Colour: used in a general model for pigment production; cc is a hypothetical albinism notation here, not proof of an identified albino degu mutation.
- D — Dilution: dd denotes a diluted coat in this convention, while D denotes the non-diluted form.
- E — Extension: used for changes in the distribution of dark and reddish pigment; ee is associated with the sand description.
- W — White patching: used for white spotting, described as dominant in the breeder model.
An asterisk indicates that the second allele is unspecified; it is not the name of another allele. Codes are a shorthand for the model, not a substitute for pedigree records, genetic testing where available, or assessment of health and behaviour.
Agouti colours
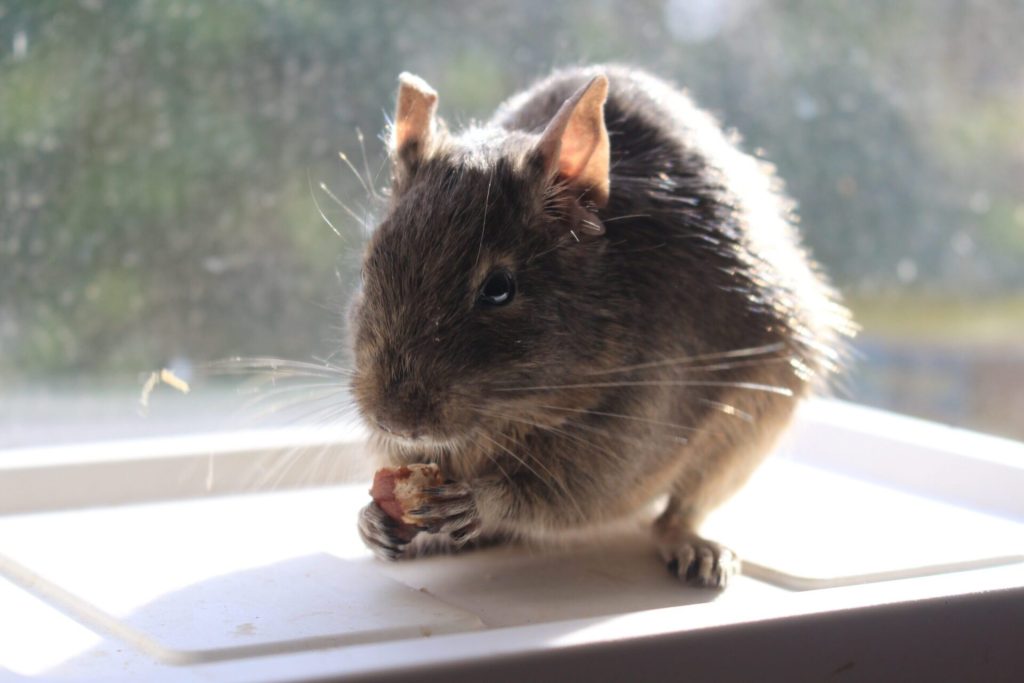
Agouti coats have banded hairs. Their appearance depends on the arrangement of lighter and darker pigment along the hair shaft.
Agouti: the natural colour
Breeder code: A* B* C* D* E* ww
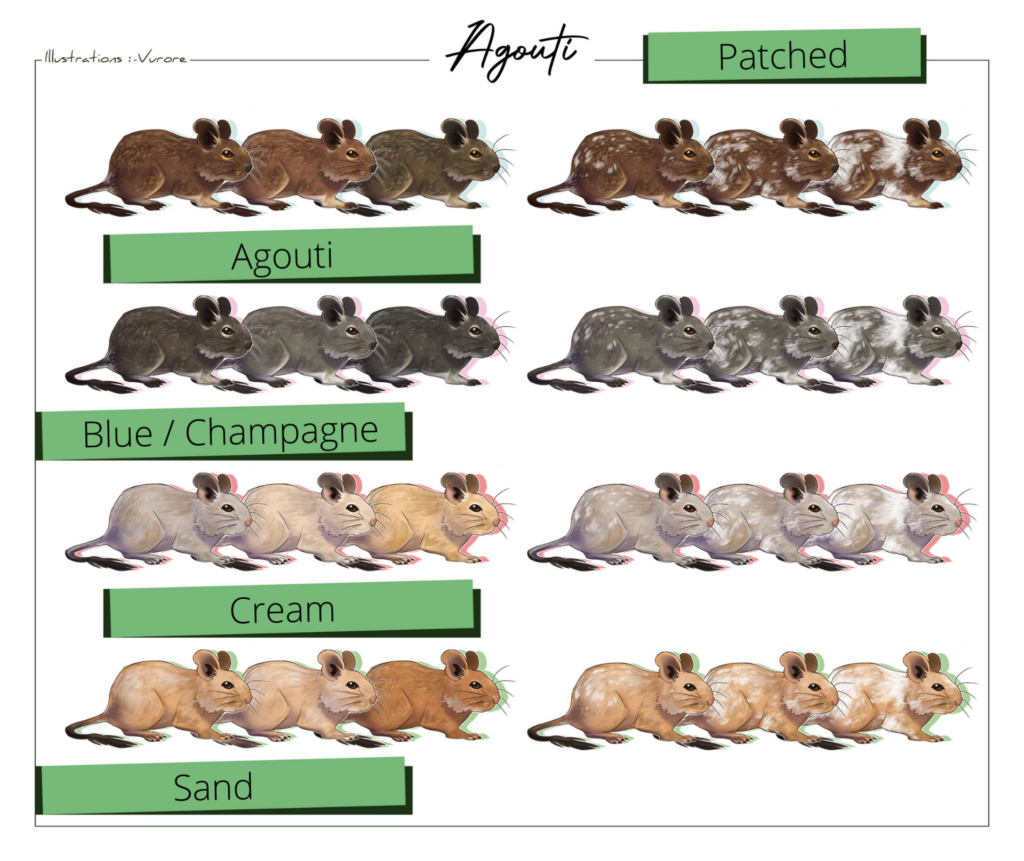
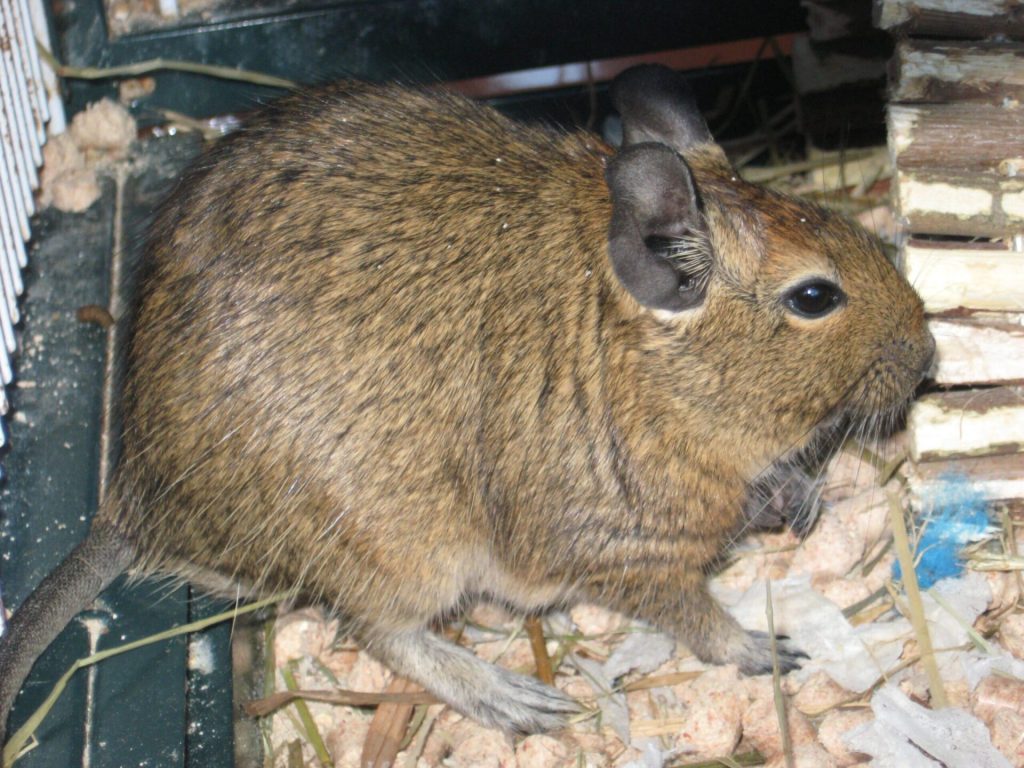
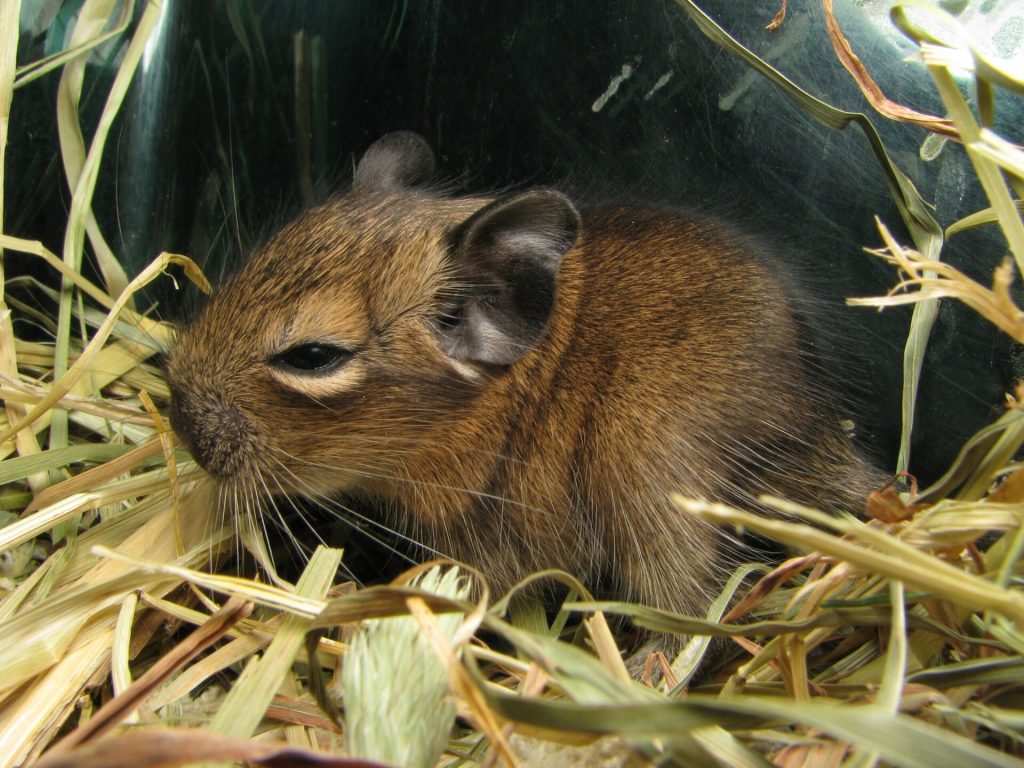
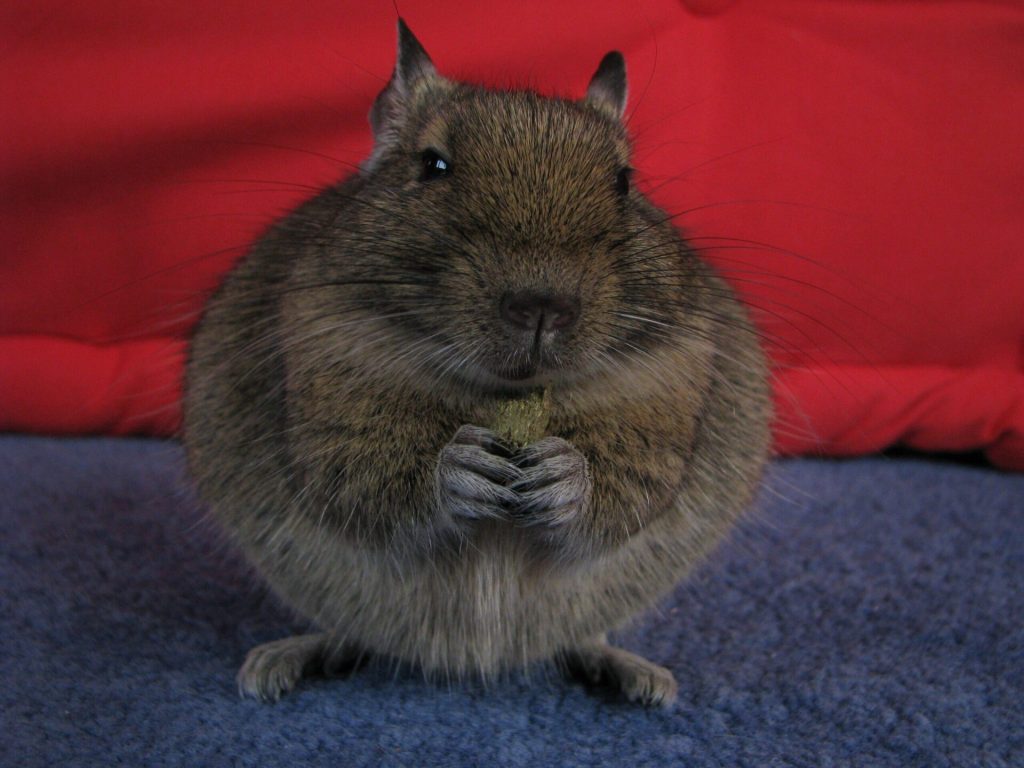
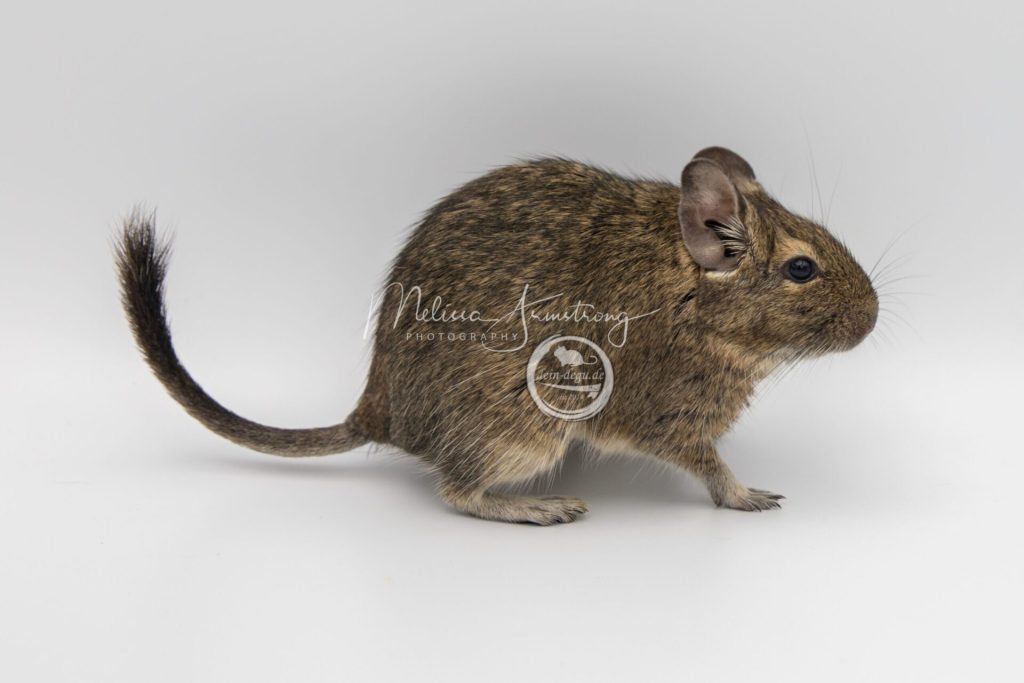
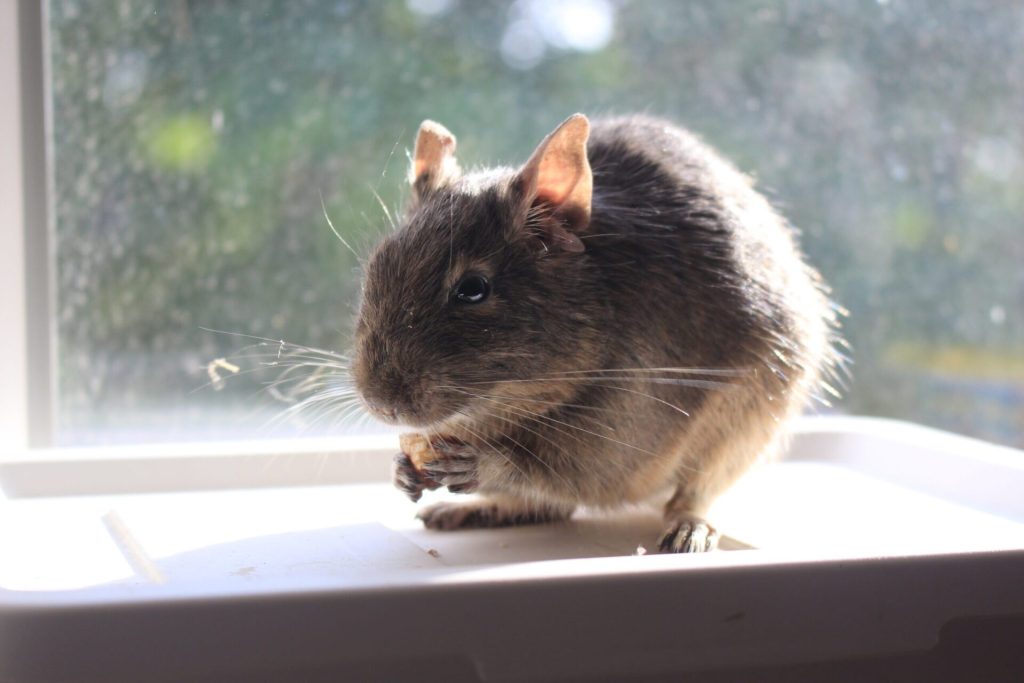
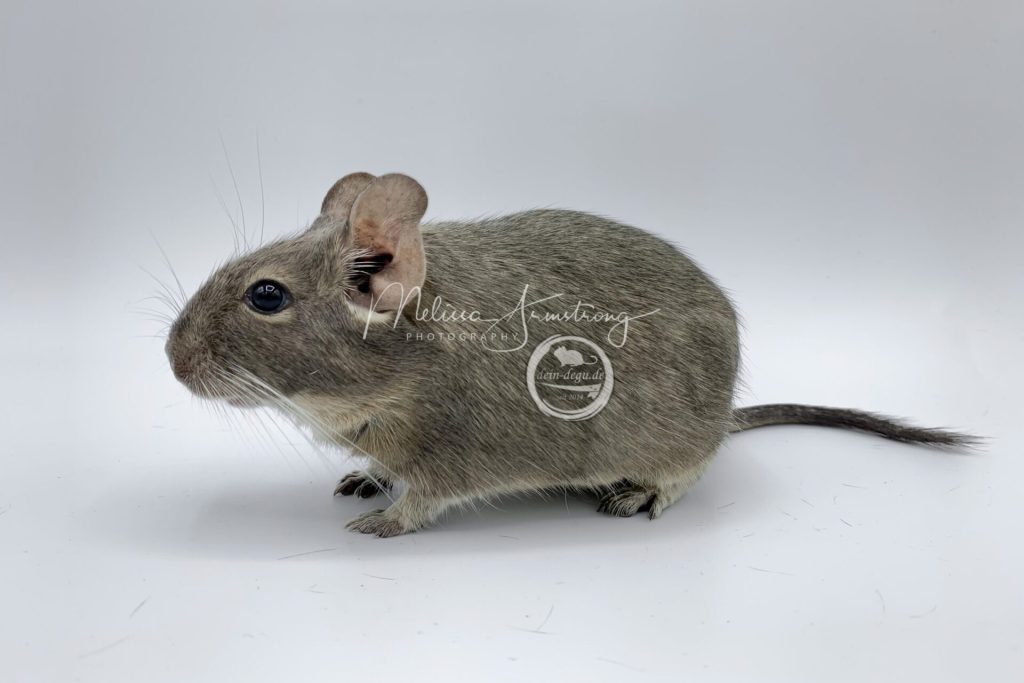
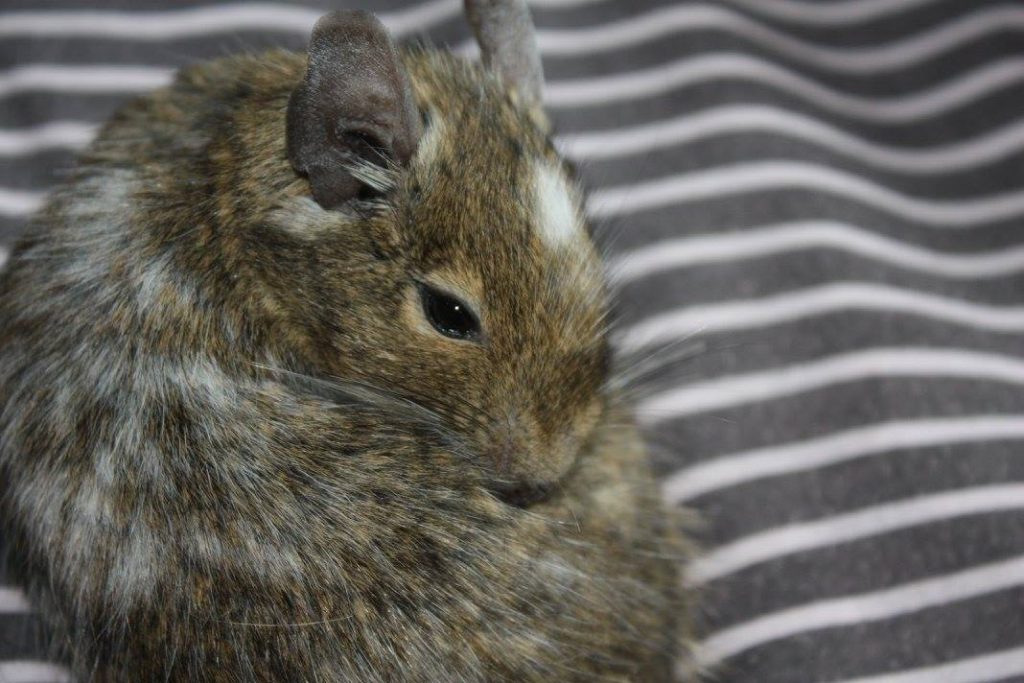
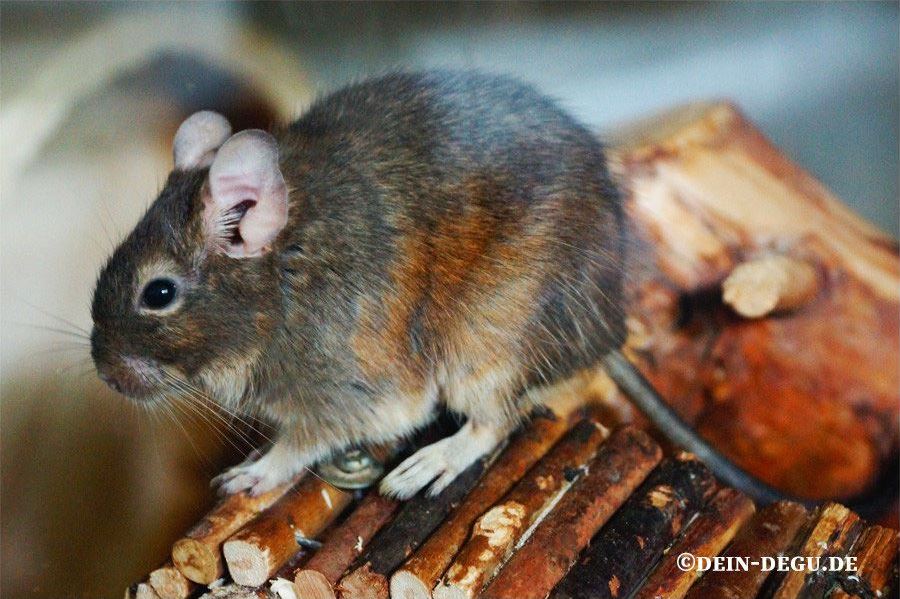
The natural agouti coat provides camouflage in the degu’s habitat. The overall appearance is brown, with dark and lighter tones. Hairs typically have a lighter pheomelanin band between darker eumelanin regions. The ears are dark, while the eye surrounds, the base of the ears and the belly are lighter beige; the feet can appear pale grey. Other agouti varieties alter this underlying pattern.
Blue agouti and champagne agouti
Breeder code: A* B* C* dd E* ww
Blue agouti degus have a predominantly light-grey appearance, sometimes with brown or cream tones. The eye surrounds, ear bases and belly remain lighter, and the feet can show grey areas. Blue was among the earlier coat variations described in captive degus and is interpreted in the breeder model as dilution of dark pigment.
The name champagne agouti is used for animals retaining a more visible pale-brown or cream band, producing warmer highlights. Naming and recognition vary among breeders; this should not be treated as a universally recognised, separate mutation. Banded blue agouti hairs should be distinguished from the more uniformly coloured hairs of non-agouti blue animals.
Sand
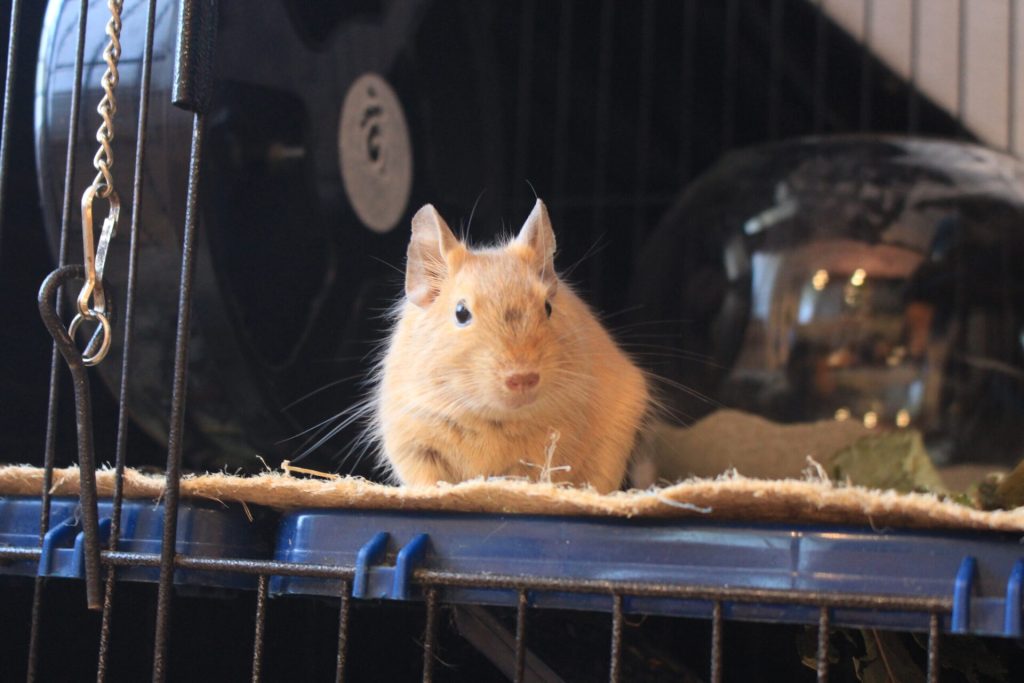
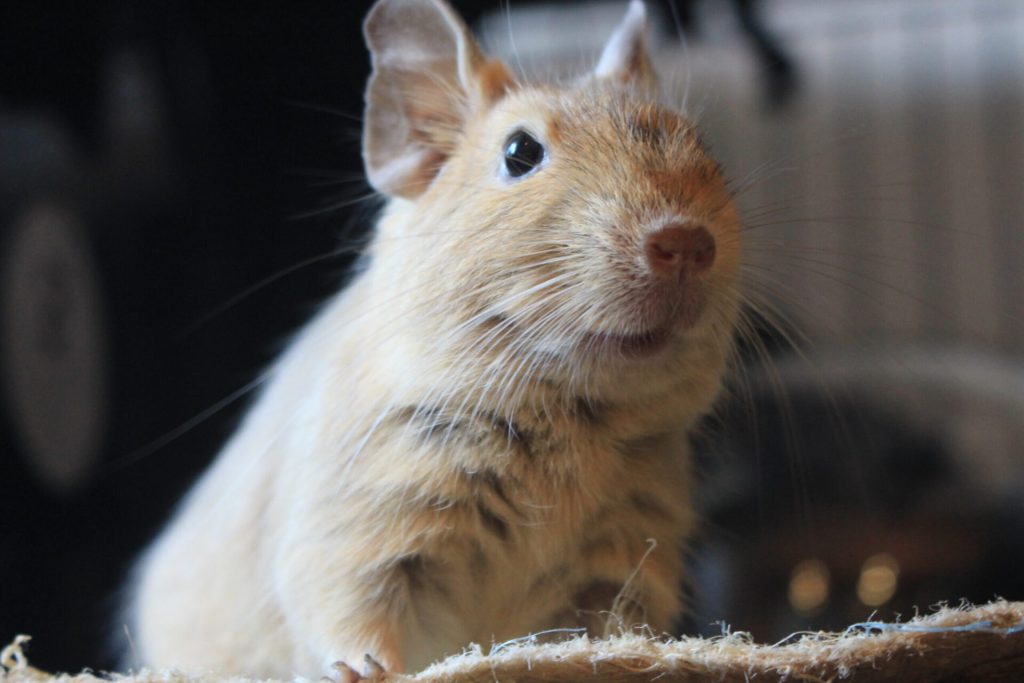
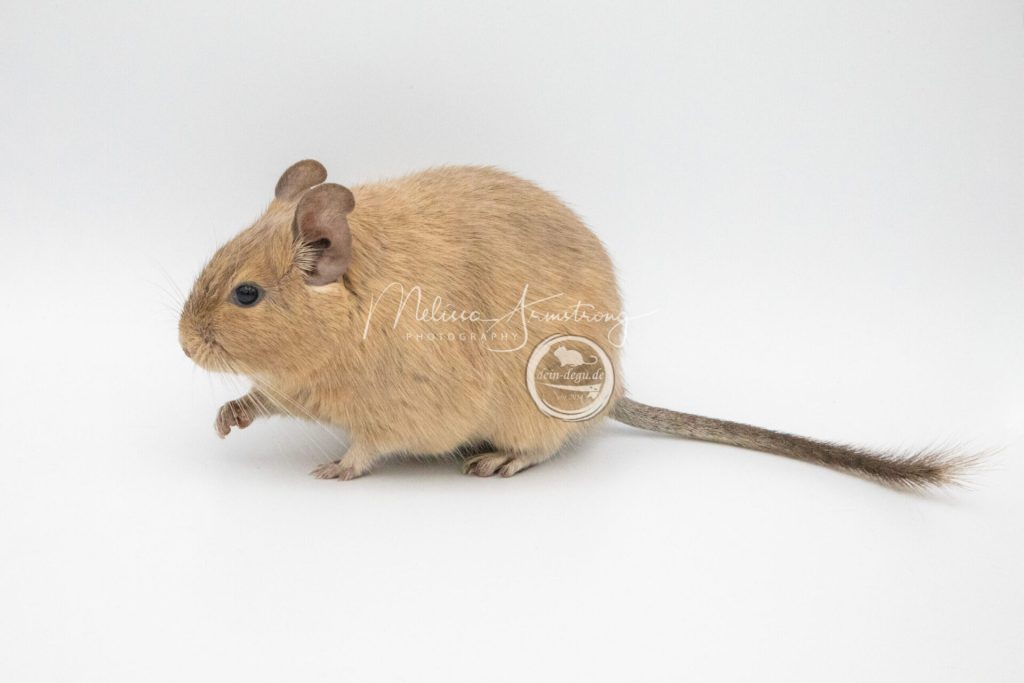
Breeder code: A* B* C* D* ee ww
Sand degus have a warm, pale reddish or sandy coat. The contrast around the eyes, ears, belly and neck can be less conspicuous than in natural agouti animals. Breeder accounts describe recessive inheritance and associate the appearance with increased pheomelanin relative to visible dark pigment along the hair.
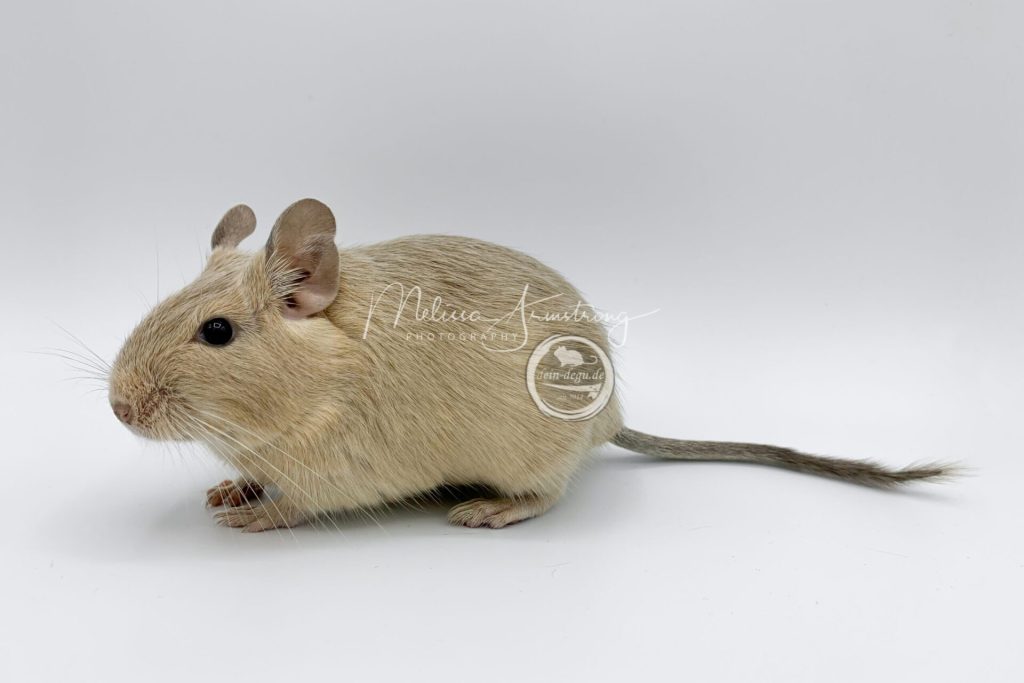
Cream
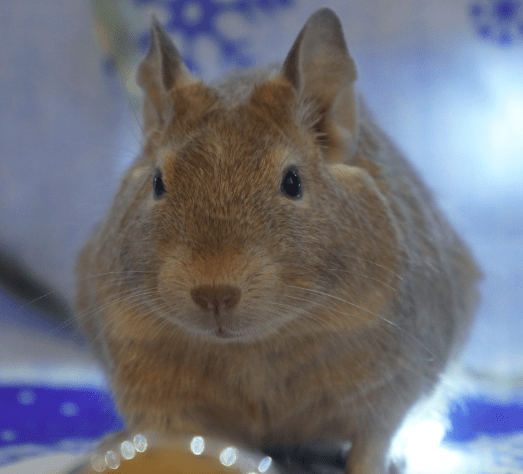
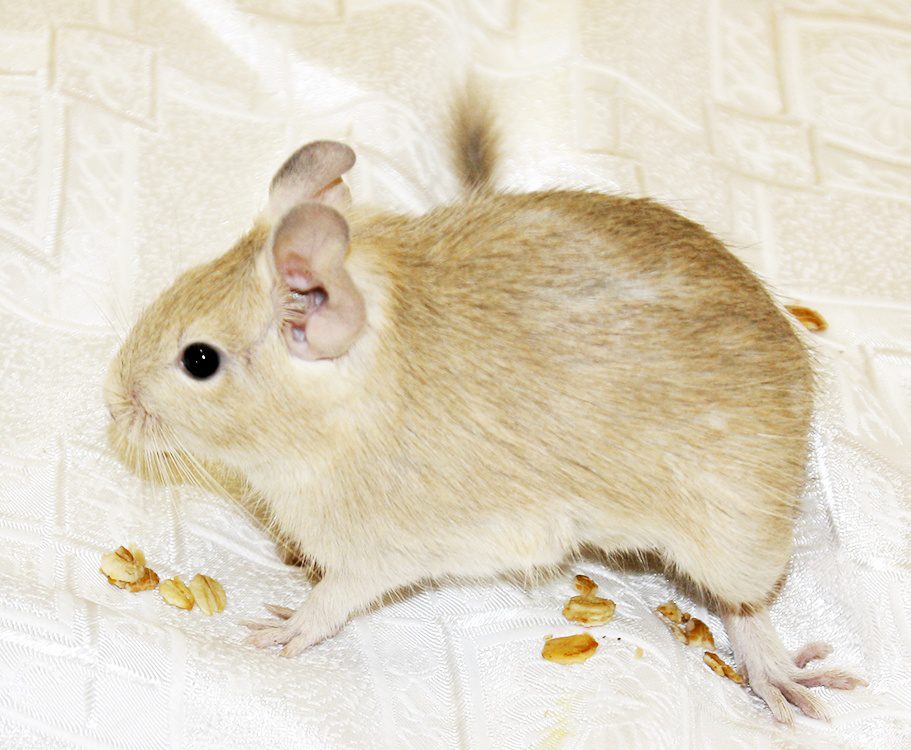
Breeder code: A* B* C* dd ee ww
Cream combines the dilution and sand descriptions in this model. The coat is lighter than sand, sometimes with champagne tones, and may darken as the animal matures, particularly where grey tips appear on the back.
The notation contains two specified recessive pairs, dd and ee, not three. Depending on parental genotypes, the desired combination may appear in later generations, but no universal rule requires a second- or third-generation cross. Closely related matings increase inbreeding risk; producing a colour does not justify compromising genetic diversity.
Non-agouti colours
Non-agouti coats lack the usual agouti banding and appear more uniform. Distinguishing some colour varieties can nevertheless be difficult from a photograph alone.
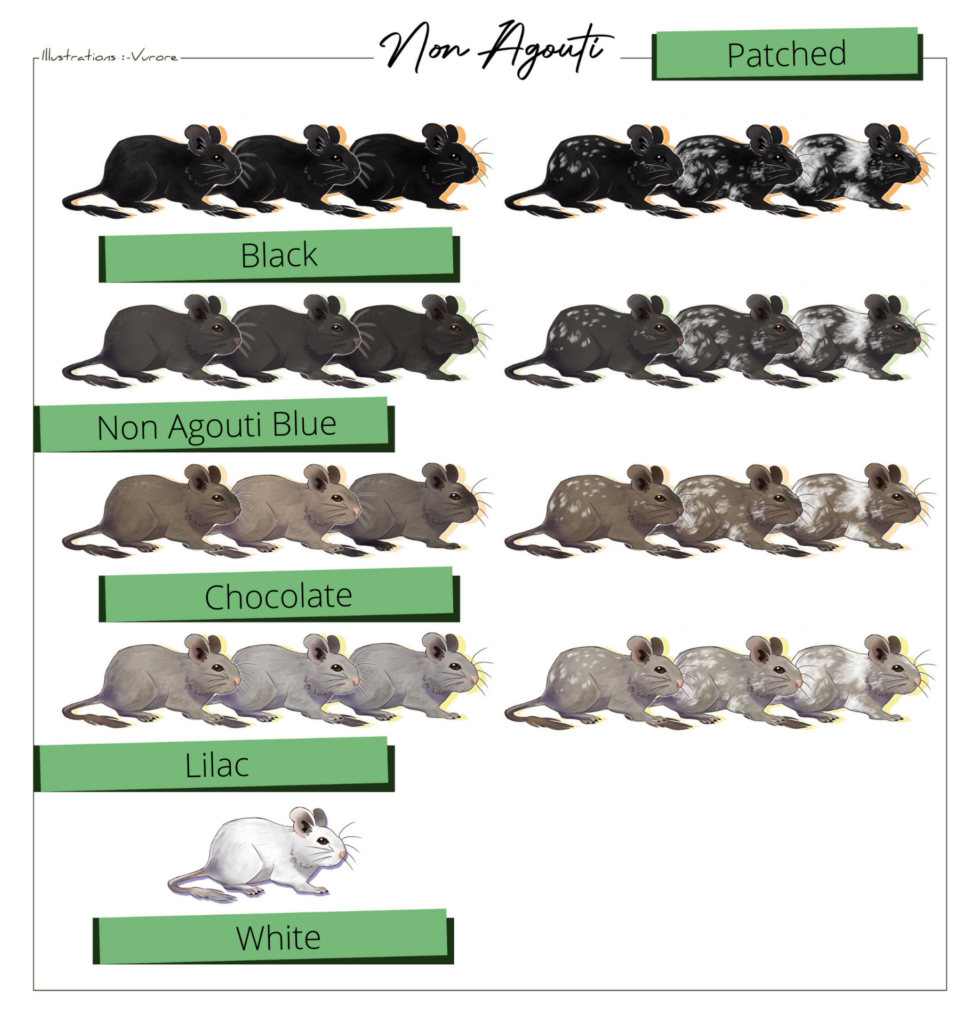
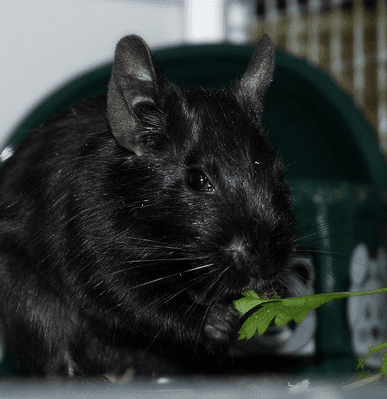
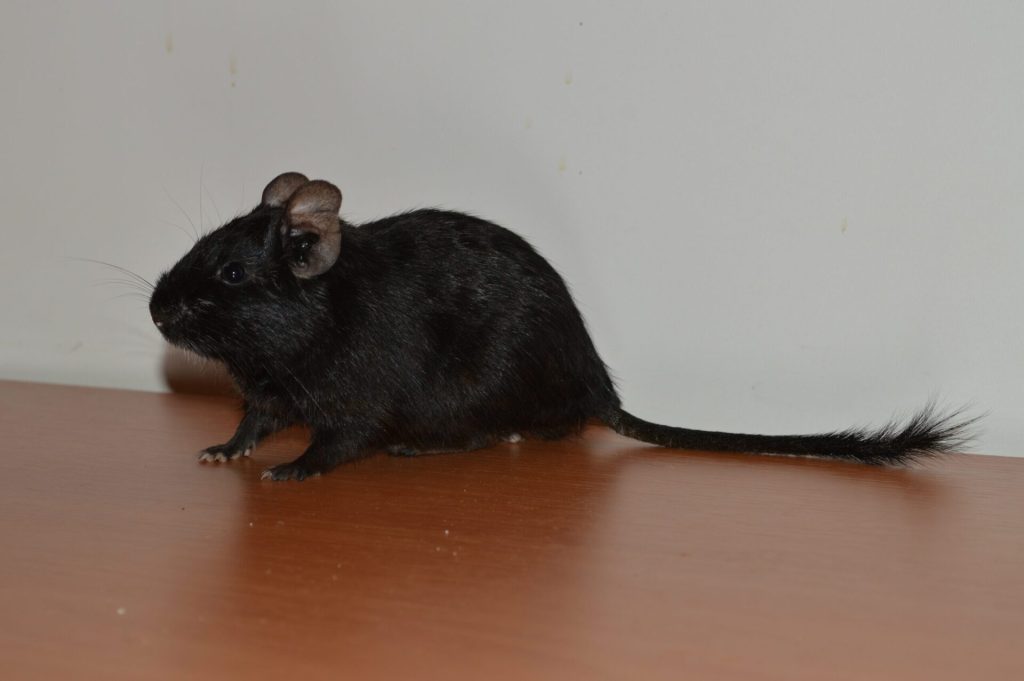
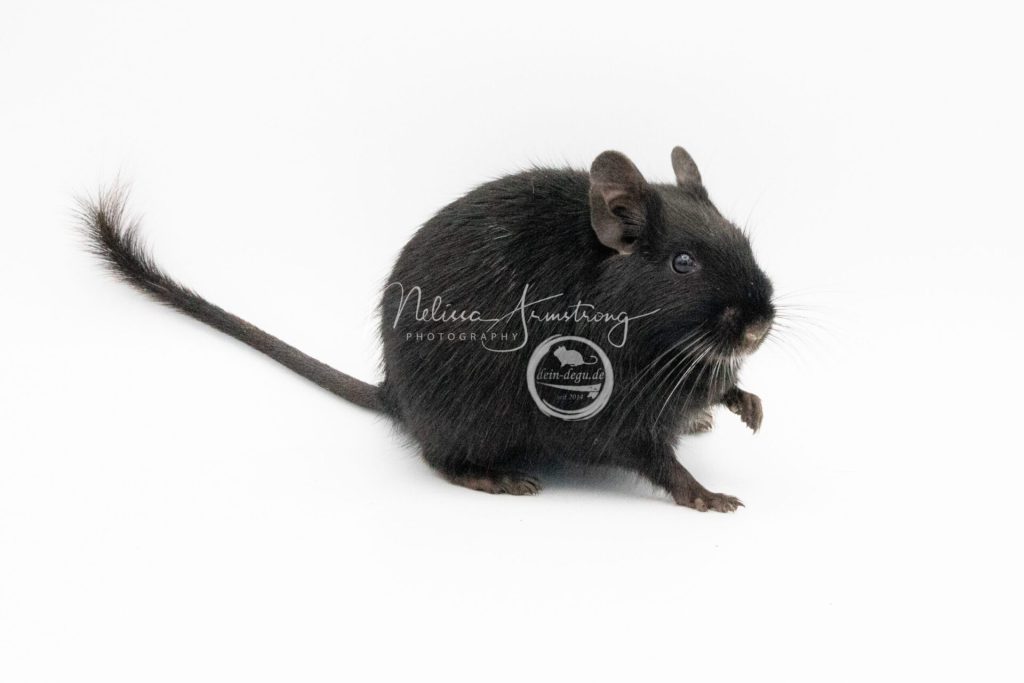
Black
Breeder code: aa B* C* D* E* ww
Black non-agouti degus often appear very dark brown rather than uniformly jet black. Dark pigment extends along the hair instead of forming the usual agouti bands. Shade and local discolouration vary, but their presence does not establish an animal’s genotype. The intense pigmentation of Ayam Cemani chickens is a different biological example and does not demonstrate the mechanism in degus.
White
White-patching model: * * C* * * W*
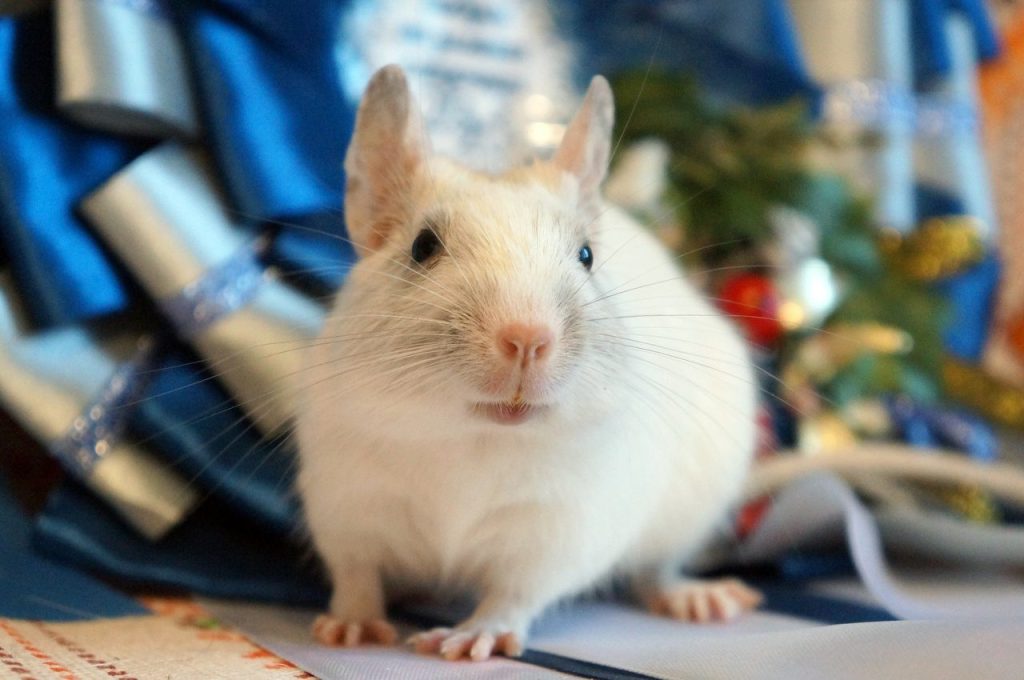
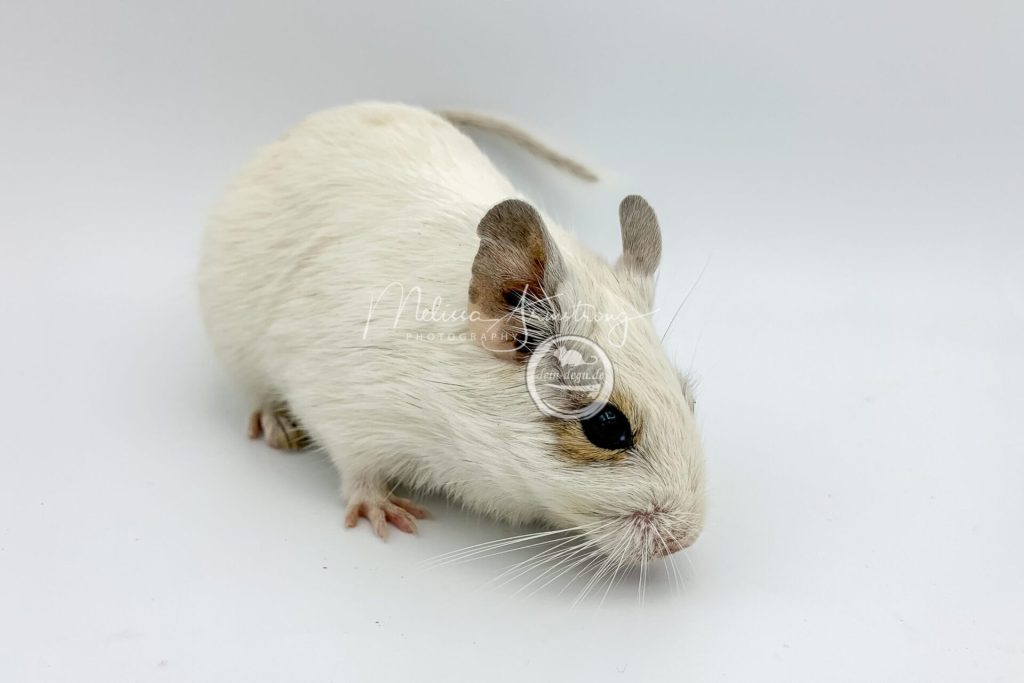
A white coat does not by itself establish albinism or extreme dilution from sand and blue. Breeder accounts distinguish extensive white spotting from rare animals whose coat becomes white as they age. Pigment may remain in the skin, ears, nails or eye surrounds; some white animals are reported to have pink skin that darkens during development.
The cited sources do not demonstrate a verified albino degu mutation, a lethal albinism allele, or a universally shortened lifespan for a presumed WW genotype. The historical article about colour inheritance in horses cannot establish these claims in degus. 3 A phenotype should not be assigned a genotype or a prognosis on that basis alone.
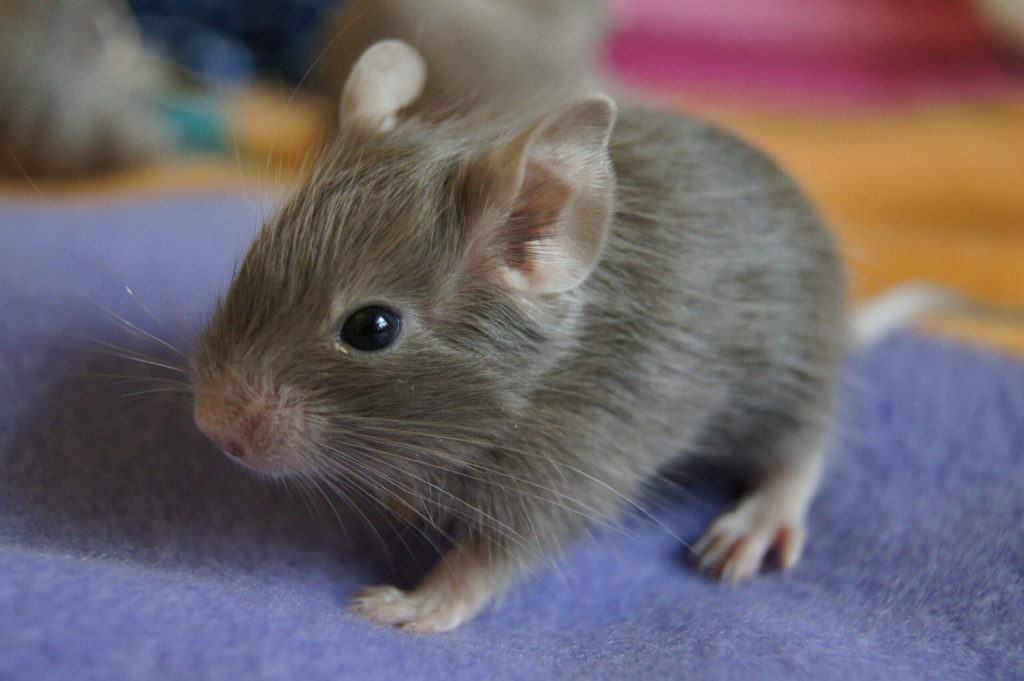
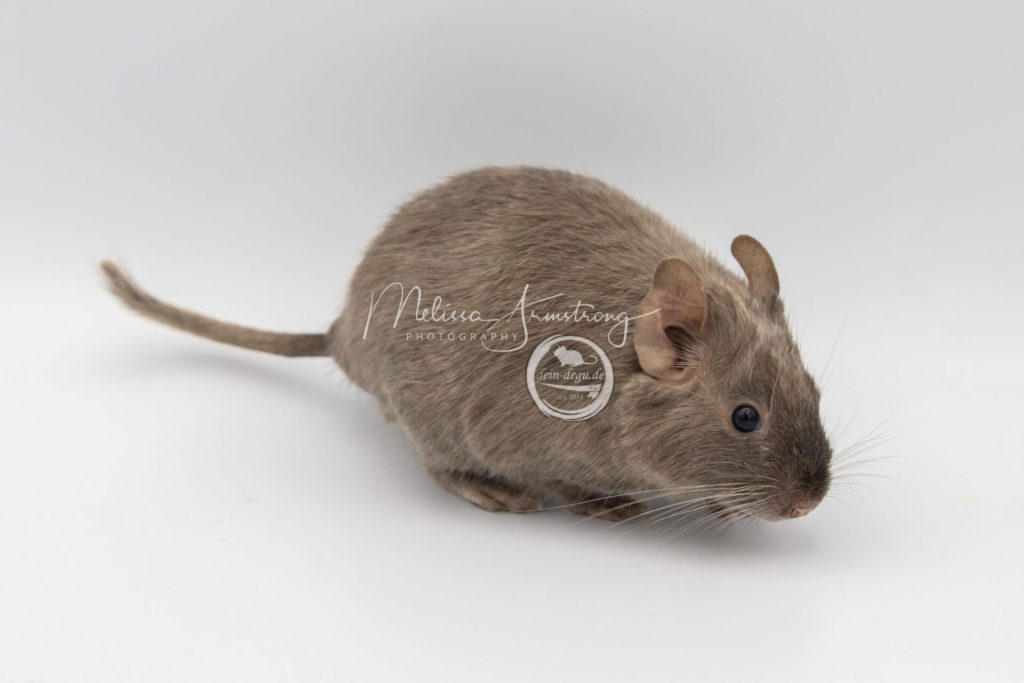
Chocolate
Historical breeder code: aa bb C* D* Ee ww
Chocolate describes a warmer, lighter brown non-agouti coat. The model attributes it to recessive brown variation, but shades vary. The specific Ee in the historical code should not be assumed from coat appearance alone.
Blue
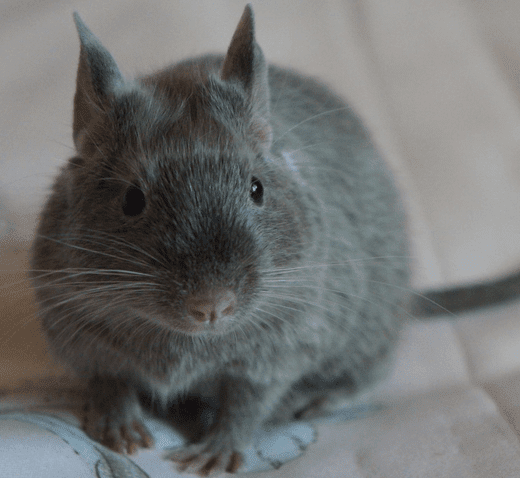
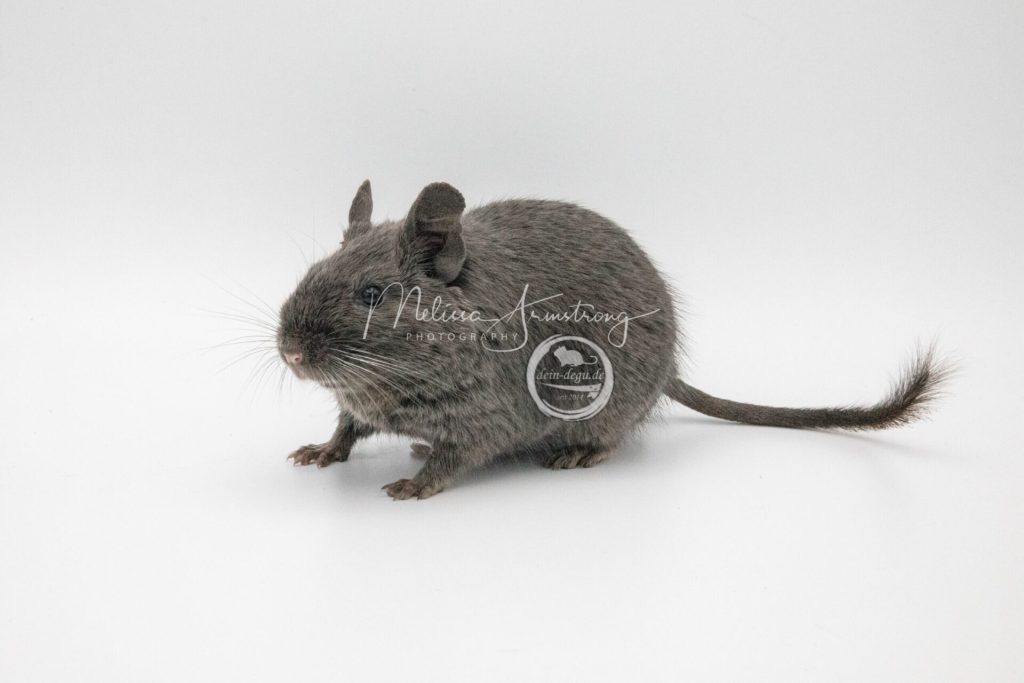
Breeder code: aa B* C* dd E* ww
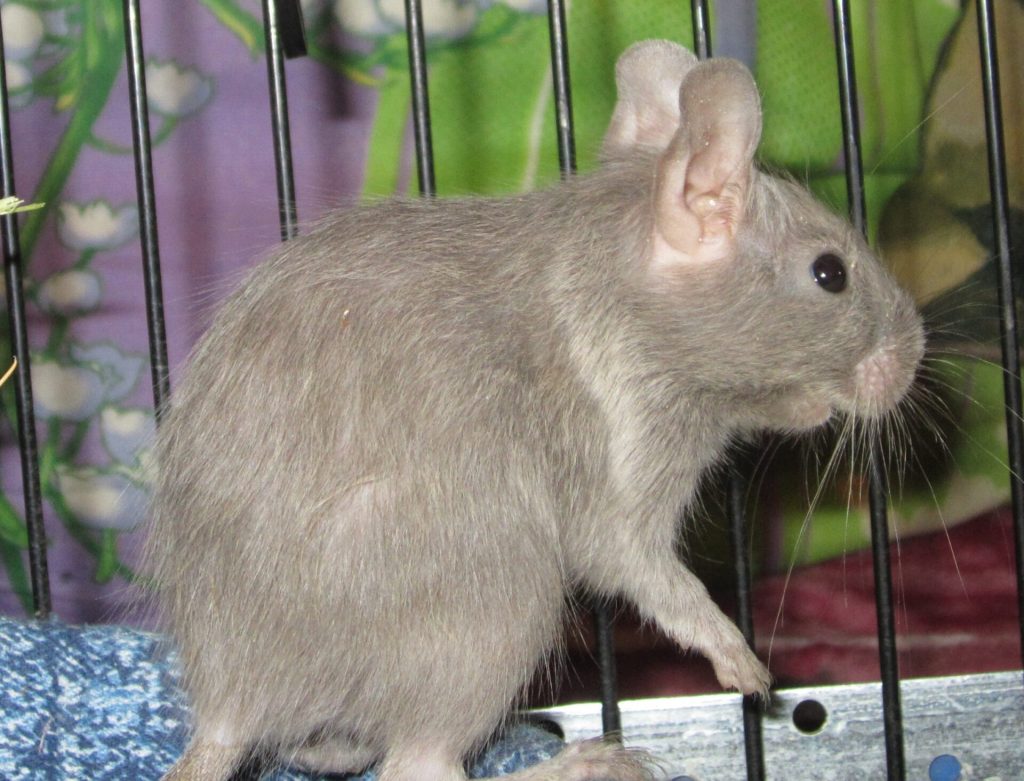
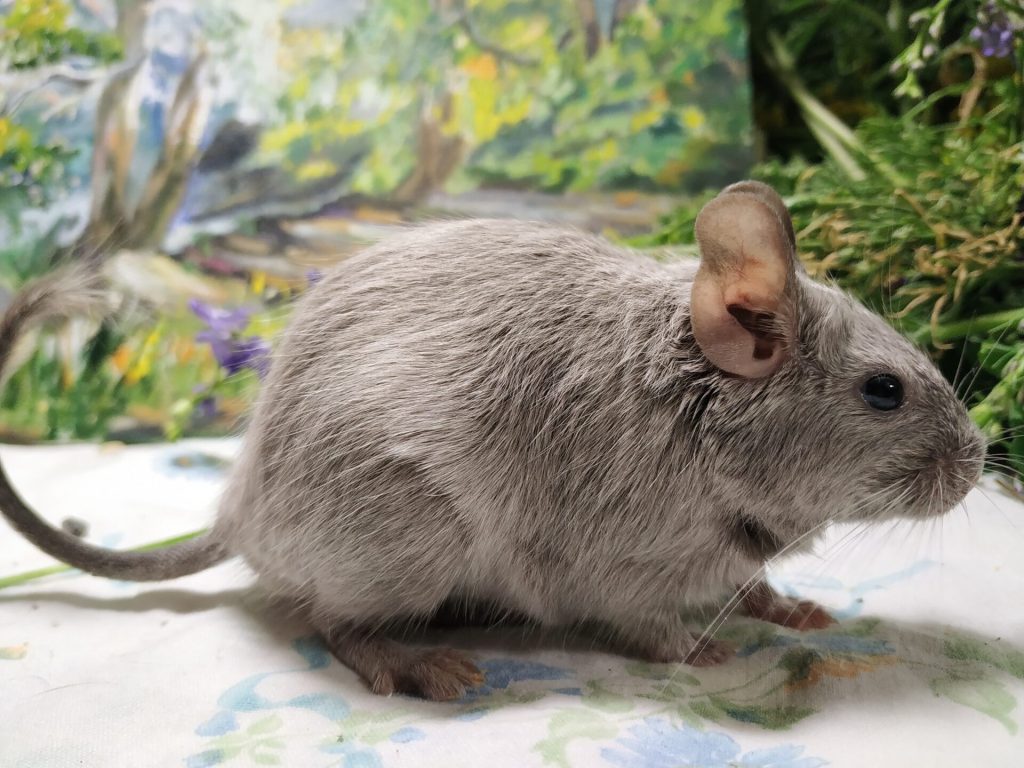
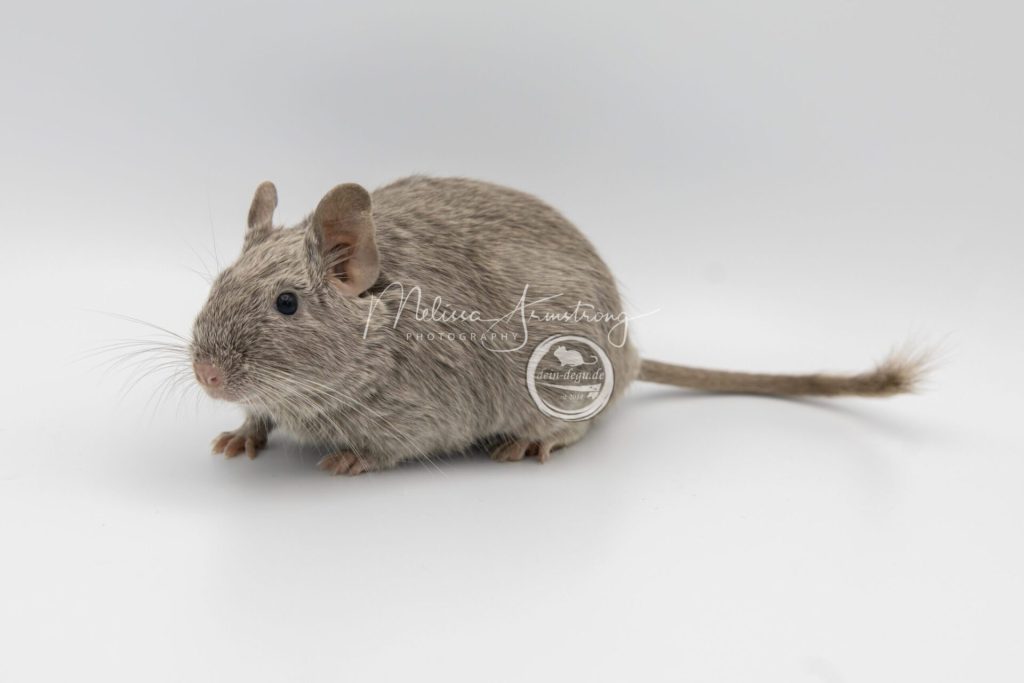
Non-agouti blue degus show a more uniform grey or blue-grey coat. Breeder terminology attributes this to dilution in a non-agouti animal. Several shades occur within the description; “blue” refers to appearance and is not itself the name of an independently demonstrated gene.
Lilac
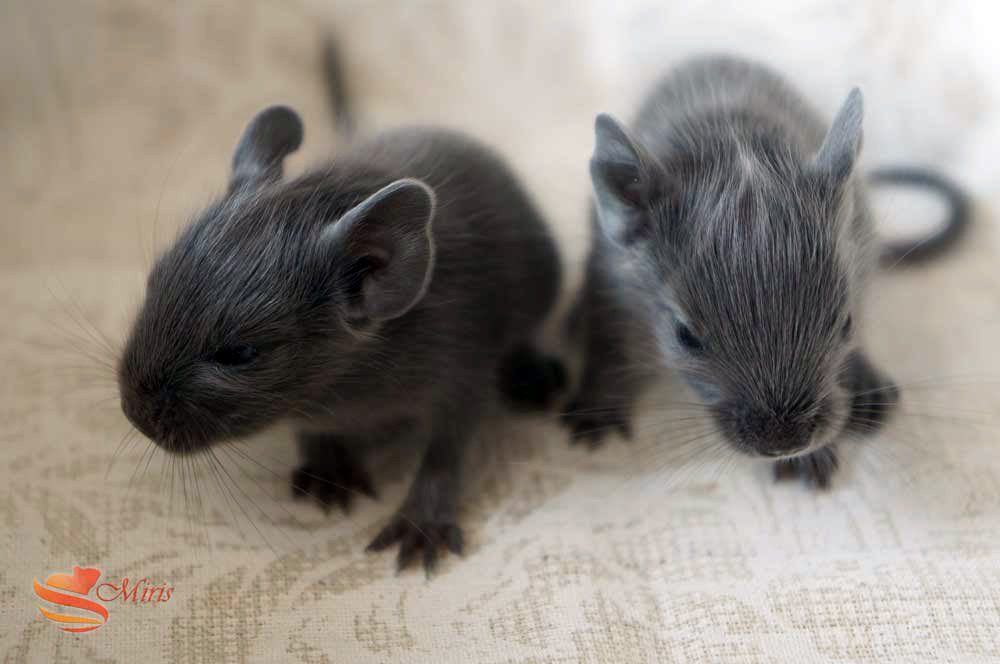
Lilac describes a relatively uncommon, pale silvery-grey non-agouti coat. Breeder accounts associate it with chocolate and blue ancestry. The original code, aa B* C* dd ee ww, does not express that same explanation: it specifies extension rather than the recessive brown pair. Without a validated degu-specific genotype, it should be retained only as a historical, inconsistent notation rather than presented as a confirmed genetic formula.
Other coat characteristics
White patching
Breeder code: * * C* * * W*
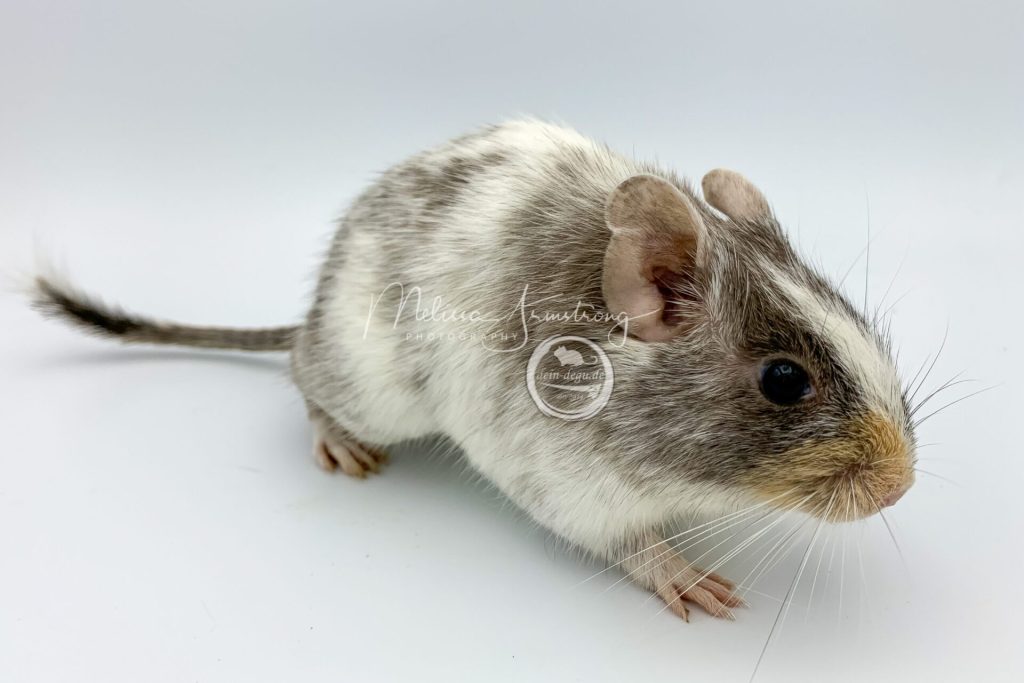
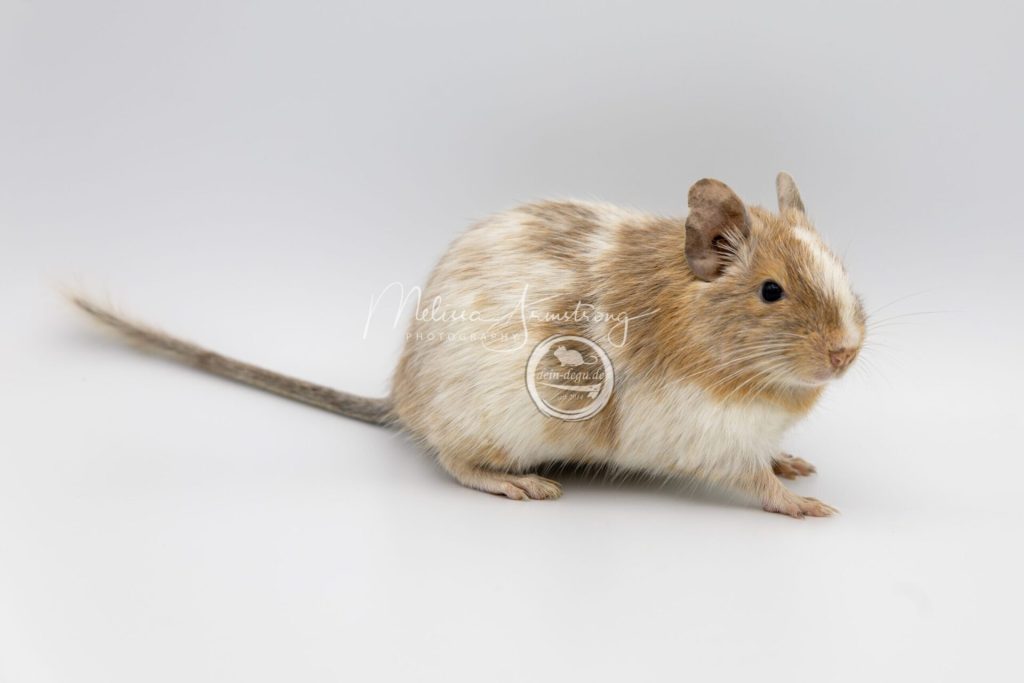
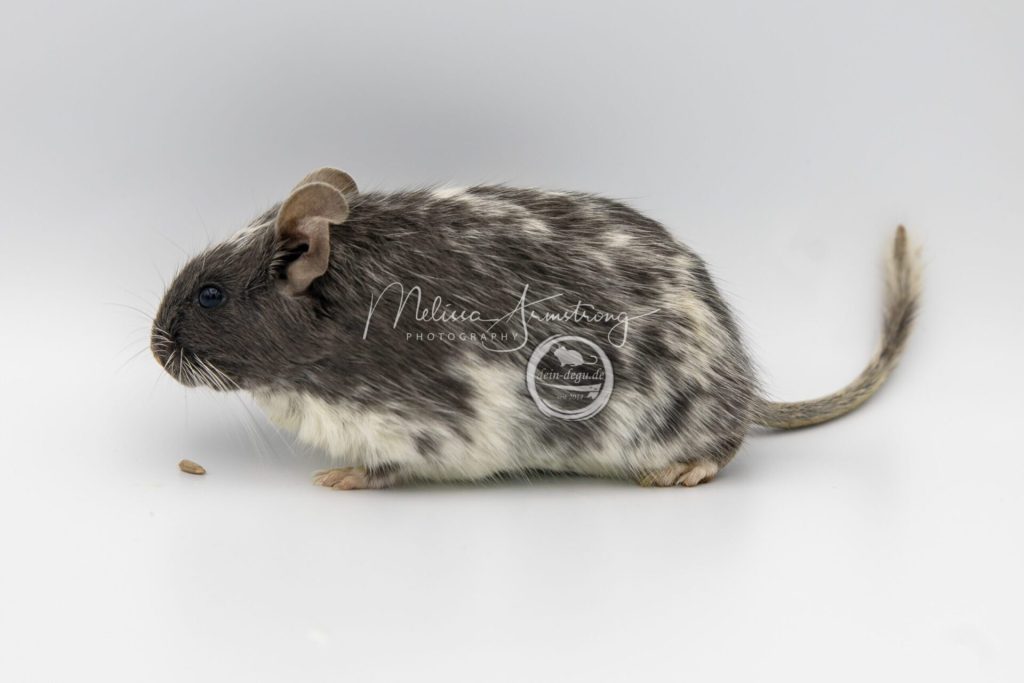
White-patched or piebald degus have unpigmented areas interrupting an otherwise coloured coat. Patching can occur with several base colours. Under the dominant model, a heterozygous patched animal is written Ww, not ww. Appearance alone does not establish whether the animal is homozygous.
The original article used the following descriptive categories:
- Patched: white markings covering less than about 40% of the body.
- Super-patched: approximately 40–70% white.
- Mega-patched: more than 70% white.
These are naming conventions rather than biological thresholds. They should not be attributed as exact current Degutopia categories: that page instead gives dot-patched below 5%, patched 5–50%, strongly patched 50–80%, and super-patched above 80%. Terminology therefore needs to be specified when comparing descriptions. 4
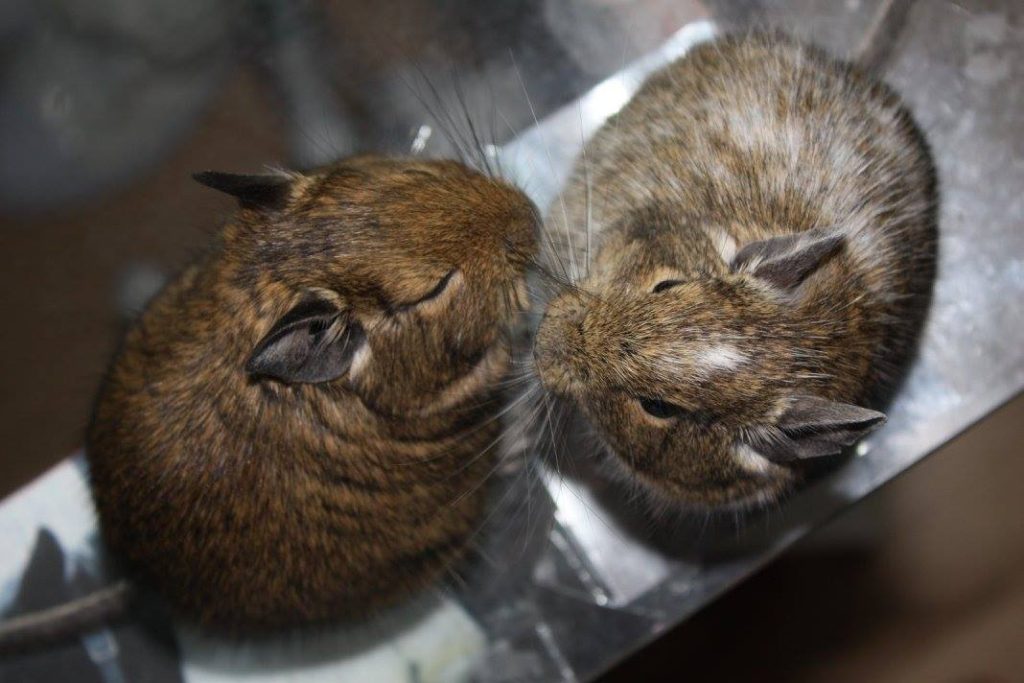
Tricolour
Breeders have reported animals described as tricolour, with three apparent coat tones. Such animals are uncommon in the cited breeder accounts, and those accounts do not establish a complete genetic explanation or predictable litter outcome. The photographs document appearance rather than a confirmed new genetic mechanism. 5
Sources
Biologie de la peau (n.d.). Les mélanines. Original website reference; the cited page is no longer available.
Montagutelli, X. & Abitbol, M. (2004). Utilisation des lignées congéniques chez la souris. médecine/sciences, 20(10), 887-893. https://doi.org/10.1051/medsci/20042010887
Castle, W. E. (1948). THE ABC OF COLOR INHERITANCE IN HORSES. Genetics, 33(1), 22-35. https://doi.org/10.1093/genetics/33.1.22
Degutopia (n.d.). Degu Colour Varieties. https://www.degutopia.co.uk/degucolours.htm
Dein-Degu (n.d.). Colors and piebalds. https://www.dein-degu.de/english/degu-facts/colours/
MedlinePlus Genetics (n.d.). Is eye color determined by genetics?. https://medlineplus.gov/genetics/understanding/traits/eyecolor/
National Human Genome Research Institute (n.d.). Codominance. https://www.genome.gov/genetics-glossary/Codominance