Degus belong to the family Octodontidae, a South American group distributed in Chile, Argentina and Bolivia. The historical Peruvian record should not be treated as a confirmed natural occurrence. The genus Octodon includes five named living species, including O. ricardojeda, formally described in a paper first published online in December 2020.
Taxonomic totals depend on the source and date. The Mammal Diversity Database consulted for this revision lists eight genera and 17 species in the family, including the extinct Octomys rosiae; the other 16 are listed as living. Its checklist includes the newly described 2026 genus and species Apnoctomys conicetorum. Older statements of 13 species, or that O. ricardojeda is not formally recognised, are outdated.
Octodontidae: classification and diversity
Taxonomic outline
| Kingdom | Animalia |
| Phylum | Chordata |
| Class | Mammalia |
| Order | Rodentia (rodents) |
| Suborder | Hystricomorpha |
| Infraorder | Hystricognathi |
| Family | Octodontidae |
| Genera (8) | Aconaemys, Apnoctomys, Octodon, Octodontomys, Octomys, Pipanacoctomys, Spalacopus, Tympanoctomys |
| Species (current checklist) | Aconaemys fuscus, Aconaemys porteri, Aconaemys sagei, Octodon degus, Octodon bridgesii, Octodon lunatus, Octodon pacificus, Octodon ricardojeda, Apnoctomys conicetorum, Octodontomys gliroides, Octomys mimax, Pipanacoctomys aureus, Tympanoctomys loschalchalerosorum, Spalacopus cyanus, Tympanoctomys barrerae, Tympanoctomys kirchnerorum, Octomys rosiae (extinct) |
| Historically listed subspecies | Spalacopus cyanus cyanus, Spalacopus cyanus maulinus, Spalacopus cyanus poeppigii |
The table follows the current MDD arrangement. Salinoctomys loschalchalerosorum is listed there as Tympanoctomys loschalchalerosorum, while Pipanacoctomys aureus remains in its own genus. Other research has proposed placing the latter in Tympanoctomys; genus boundaries should therefore be attributed to a named classification. The three Spalacopus cyanus subspecies shown are historical names retained from the original article, not a complete current subspecies inventory for the family.
General characteristics
Octodontids are relatively small, rat-like rodents. Size varies by species; figures around 20cm for body length and 300g are descriptive examples rather than limits for the whole family. Head shape, ear size, tail length and the development of a terminal tail tuft also vary. Whiskers contribute to sensory exploration.
The limbs are relatively short. In degus the fifth digit is reduced, especially on the forefoot, where it bears a nail rather than the usual claw; the simplified “four toes in front, five behind, all with claws” description overlooks this detail. Fur is generally dense, with an undercoat; many species are greyish or brownish with paler underparts, whereas Spalacopus cyanus is conspicuously dark. Some have stiff hairs extending around the hind toes.
Tail skin loss during a predator encounter must not be described as harmless shedding of the tuft: in pet degus it is a serious injury. Never handle an animal by its tail.
The family includes surface-active, burrowing and predominantly subterranean forms. Diets are largely herbivorous, and some species are considered crop pests locally. Activity schedules and social systems vary; neither nocturnality nor colony living is a rule for every octodontid. Common degus provide a well-studied example of complex social behaviour.
Habitats and geographical distribution
Octomys is associated with surface activity, while Octodontomys, Octodon and Tympanoctomys use burrows to varying degrees. Aconaemys is more fossorial, and Spalacopus is especially specialised for subterranean life. These categories describe a continuum rather than identical behaviour within each genus.
Octomys and Tympanoctomys occur in arid and semi-arid parts of central-western Argentina. Spalacopus occurs in central Chile. Octodon and Aconaemys occur in Chile and south-western Argentina, with species-specific distributions in scrub, grassland or forest environments. Octodontomys occurs in open habitats of north-western Argentina, south-western Bolivia and northern Chile. The recently described Apnoctomys is from the hilly Chaco of central Argentina.
Evolutionary history
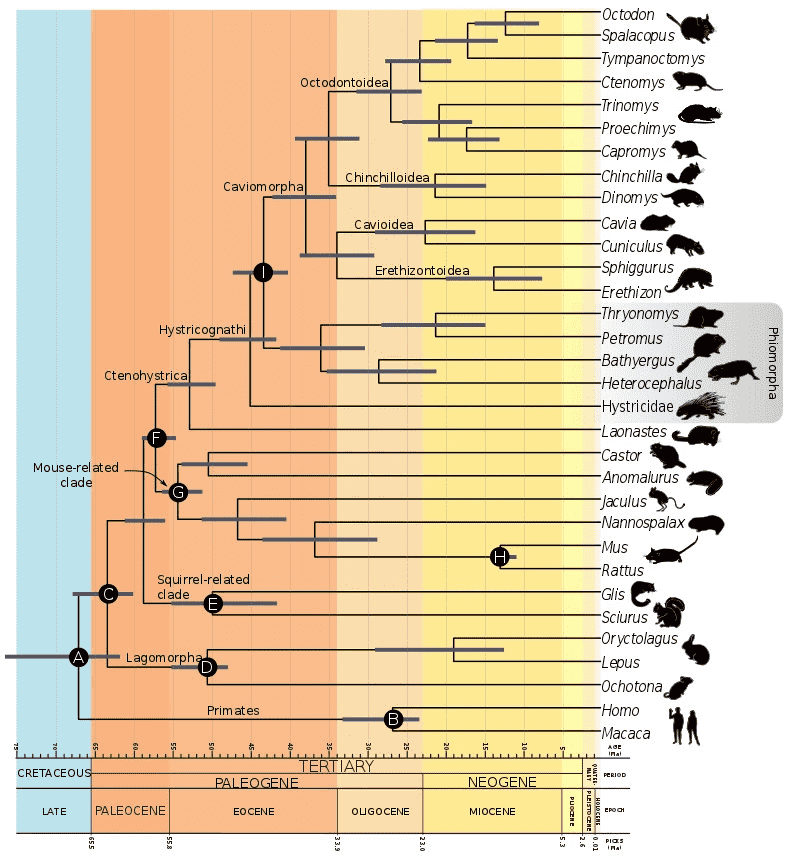
Octodontid diversification forms part of the wider radiation of South American caviomorph rodents. Molecular studies place relevant divergences in the Miocene, but dates depend on the lineage, calibration and analysis. The earlier figure of 8.8 million years, in the Tortonian stage of the late Miocene, should be read as an estimate for a particular evolutionary node, not a precise date at which every present-day species originated.
The genus Octodon
Etymology
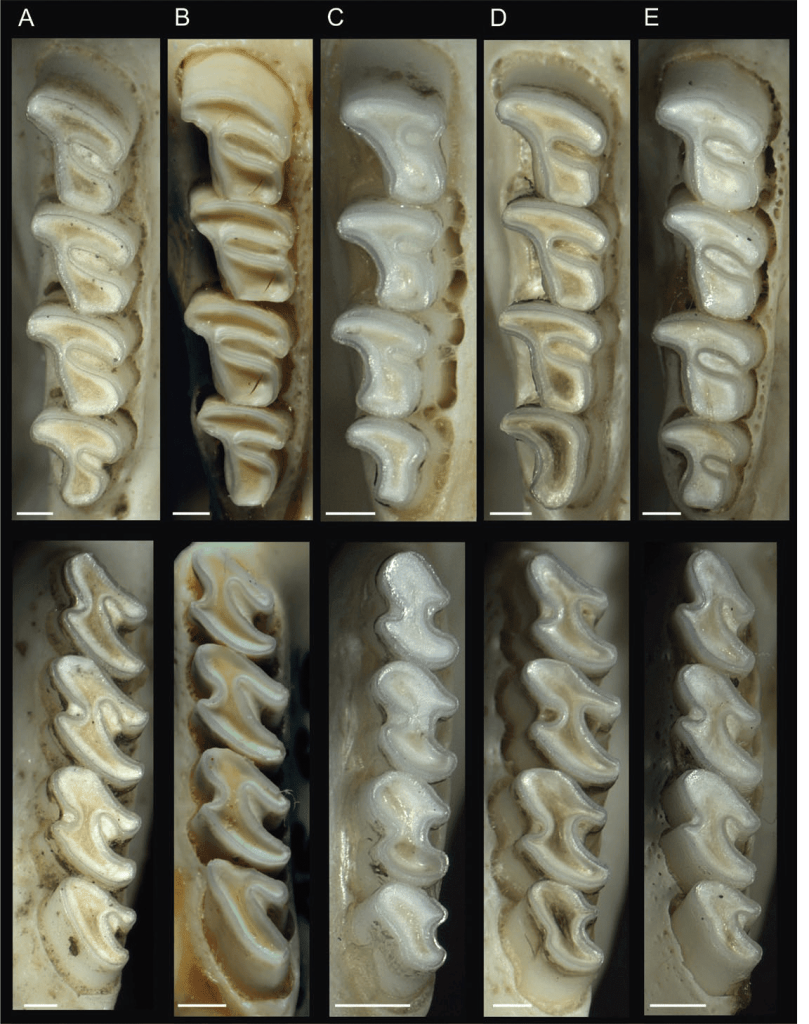
Octodon derives from Greek elements meaning “eight” and “tooth”, referring to the figure-of-eight pattern of the cheek teeth. In English these animals are called degus; “degu” without further qualification usually means O. degus.
Classification
| Kingdom | Animalia |
| Phylum | Chordata |
| Class | Mammalia |
| Order | Rodentia (rodents) |
| Suborder | Hystricomorpha |
| Infraorder | Hystricognathi |
| Family | Octodontidae |
| Genus | Octodon |
| Species | Octodon degus, Octodon bridgesii, Octodon lunatus, Octodon pacificus, Octodon ricardojeda |
History of the named species
Molina described the common degu in 1782 as Sciurus degus; the modern combination is Octodon degus. Names associated with its taxonomic history include clivorum (Thomas, 1927), cumingii (Bennett, 1832), getulinus (Poeppig, 1829), pallidus (Wagner, 1845) and peruana (Tschudi, 1845). Their historical use does not imply five additional currently accepted species.
Thomas distinguished O. d.degus and O. d.clivorum, while later treatments regarded the species as monotypic. The claim that no subspecies have subsequently been recognised is outdated: Cadenillas and D’Elía’s 2021 revision distinguished northern and southern morphotypes, designated a neotype and described a northern subspecies.
Waterhouse described O. bridgesii in 1844, not 1945. Both “bridgesi” and “bridgesii” occur in the literature; the current MDD uses the latter. The historical type-locality discussion concerns Río Teno, Colchagua, Chile, not a territory newly created in 1927.
Osgood described O. lunatus in 1943, with Olmué, Valparaíso, as its type locality. Its distinction from O. bridgesii was later debated. Chromosomal and molecular studies support differentiation, but a C-band karyotype study should not be mislabelled simply as a DNA-sequence analysis. Hutterer described O. pacificus from Isla Mocha in 1994.
D’Elía and colleagues described O. ricardojeda in a paper first published online on 10 December 2020 and assigned to the 2021 journal volume. This explains the two dates seen in references; it is not an unnamed or unofficial species.
Distribution and species limits
The genus is not restricted to Chile: records from Argentina, including Neuquén, have played an important role in revising its taxonomy. Archaeological material, predator pellets and living specimens provide different kinds of evidence and must be interpreted with their identification history in mind. Some southern populations formerly assigned to O. bridgesii are now assigned to O. ricardojeda.
The old Peruvian record associated with the name peruana was considered likely erroneous in the 2015 South American mammal reference. It should not be used to extend the genus’s confirmed wild distribution to Peru.
Phylogenetic work supports the distinct status of O. pacificus, but mitochondrial and nuclear trees do not always recover identical relationships with other southern forms. “Very similar genes” is insufficient to resolve a species boundary on its own.
Continuing taxonomic research
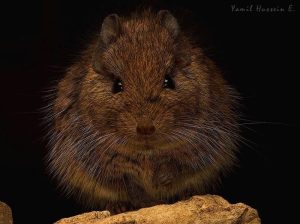
The 2021 studies found evidence that diversity within Octodon remains underestimated. Coastal populations historically assigned to O. bridgesii, including material from the Biobío and Maule regions, differ from other populations. Their relationship to O. lunatus and other lineages requires an integrated evaluation of morphology, chromosomes, multiple genetic markers and population sampling.
Candidate lineages identified by a species-delimitation method are not automatically newly named species. Different methods can recover different numbers. Reliable revisions require broad sampling and careful comparison within and between populations; further research may change both species limits and the family’s genus-level arrangement.
Sources
Mammal Diversity Database / American Society of Mammalogists (2026). Octodontidae. Current taxonomic checklist, consulted 20 October 2026. https://www.mammaldiversity.org/family/octodontidae/
D’Elía, G., Teta, P., Verzi, D. H., Cadenillas, R., & Patton, J. L. (2021). A new living species of degu, genus Octodon (Hystricomorpha: Octodontidae). Journal of Mammalogy, 102(1), 139–154; first published online 10 December 2020. https://doi.org/10.1093/jmammal/gyaa143
Cadenillas, R., & D’Elía, G. (2021). The number of species of degus (genus Octodon) is currently underestimated: An appraisal of species limits and their phylogenetic relationships (Rodentia: Hystricomorpha: Octodontidae). Molecular Phylogenetics and Evolution, 159, 107111. https://doi.org/10.1016/j.ympev.2021.107111
Cadenillas, R., & D’Elía, G. (2021). Taxonomic revision of the populations assigned to Octodon degus (Hystricomorpha: Octodontidae): With the designation of a neotype for Sciurus degus G. I. Molina, 1782 and the description of a new subspecies. Zoologischer Anzeiger, 292, 14–28. https://doi.org/10.1016/j.jcz.2021.02.008
Suárez-Villota, E. Y., et al. (2016). Filling phylogenetic gaps and the biogeographic relationships of the Octodontidae (Mammalia: Hystricognathi). Molecular Phylogenetics and Evolution, 105, 96–101. https://doi.org/10.1016/j.ympev.2016.08.015
Voloch, C. M., Vilela, J. F., Loss-Oliveira, L., & Schrago, C. G. (2013). Phylogeny and chronology of the major lineages of New World hystricognath rodents: Insights on the biogeography of the Eocene/Oligocene arrival of mammals in South America. BMC Research Notes, 6, 160. https://doi.org/10.1186/1756-0500-6-160
Upham, N. S., & Patterson, B. D. (2015). Evolution of caviomorph rodents: A complete phylogeny and timetree for living genera. In Biology of Caviomorph Rodents: Diversity and Evolution, pp. 63–120. SAREM. https://n8u.org/pubs/
Patton, J. L., Pardiñas, U. F. J., & D’Elía, G. (eds.) (2015). Mammals of South America, Volume 2: Rodents. University of Chicago Press; historical taxonomic reference. https://www.biodiversidad.gob.ec/wp-content/uploads/downloads/2019/08/Patton_2015.pdf
Woods, C. A., & Boraker, D. K. (1975). Octodon degus. Mammalian Species, 67, 1–5. https://doi.org/10.2307/3503820
Hutterer, R. (1994). Island rodents: A new species of Octodon from Isla Mocha, Chile (Mammalia: Octodontidae). Zeitschrift für Säugetierkunde, 59, 27–41. https://www.zobodat.at/pdf/Zeitschrift-Saeugetierkunde_59_0027-0041.pdf
Teta, P., et al. (2026). A new genus and species of octodontid rodent from the hilly Chaco of central Argentina (Rodentia: Octodontidae). Vertebrate Zoology, 76, 361–380. https://doi.org/10.3897/vz.76.e187462
Verzi, D. H., et al. (2024). A new extinct desert rodent from the Holocene of South America and its bearing on the diversity of Octodontidae (Hystricognathi). Journal of Mammalogy, 105(1), 59–72; first published online 15 December 2023. https://doi.org/10.1093/jmammal/gyad106