The common degu (Octodon degus) is native to Chile. Studying its natural environment, activity, feeding and social relationships helps explain its needs in captivity. Field observations and laboratory research provide complementary information, but findings from one setting should not automatically be generalised to every population.
History and scientific study
Juan Ignacio Molina described the animal in 1782 as Sciurus degus. Later classifications changed its generic placement, and Waterhouse used the combination Octodon degus in 1848. Historical accounts also mention albino animals observed in 1967 and other unusual coat colours. Wolffsohn proposed the high-altitude form O. degus clivorum in 1927, but it has not generally been recognised as a distinct valid subspecies.1
Distributional and anatomical work expanded during the twentieth century, including Osgood’s 1943 account and Mann’s anatomical studies.1 Degus subsequently became important research animals in studies of social behaviour, diabetes and age-related processes, including Alzheimer’s-like pathology. This is a research-model role, not a statement that every degu develops the human disease.2
Geographical distribution
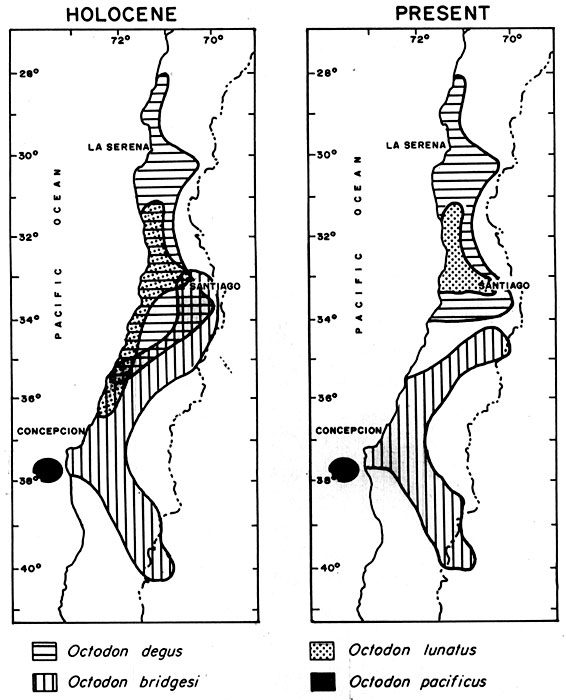
O. degus is endemic to Chile.3 Its distribution must be distinguished from that of the whole genus: Argentine degus include O. ricardojeda, formerly confused with other species. Some species’ ranges overlap, whereas O. pacificus is restricted to Mocha Island. Historical absence of reported hybrids should not be treated as proof that all species share the same territory or that hybridisation has been tested exhaustively.
Archaeological remains show that degus have long occurred in Chile. The original account cites material dated to around 200 BCE; such a date documents one archaeological occurrence, not the origin of the species.4 Degus are common in several central Chilean habitats,1 but human activities have altered distributions and contributed to local losses. This does not establish a uniform decline in every population.5
The Pacific degu was long considered possibly extinct. A dead female publicised in 2016 provided renewed evidence of its persistence, and CONAF confirmed four live animals captured and released on Mocha Island in March 2024.23 Poisons used against introduced rats can also threaten native rodents; their use does not selectively protect native degus.
Habitat and activity
Burrows and territorial structures
Wild degus are mainly active by day, often with morning and evening peaks that vary with temperature and season. Their burrow systems contain tunnels, chambers and multiple entrances, frequently near vegetation. Burrows provide shelter, nesting places and a focus for group activity.1
Sticks, stones and dung may accumulate near entrances. Older observations associated mound building with territorial marking and male status, but the function of every mound and the consequences of its destruction should not be assumed to be identical.1 A separate study examined captive degus spontaneously arranging objects into “Chinese boxes”; this is evidence about object manipulation, not direct proof that wild degus plug burrows with the same behaviour.6
Historical accounts discussed relationships among Octodon and other burrowing rodents, including the genus Ctenomys.7 Burrow sharing is specifically reported with Bennett’s chinchilla rat (Abrocoma bennettii), including observations of mothers and young using the same nest.49 This does not make the chinchilla rat an obligate parasite or establish that it cannot live without degus.
Predators and defensive behaviour
Predators influence both survival and behaviour.8 They include the culpeo fox (Lycalopex culpaeus), barn owl (Tyto alba), short-eared owl (Asio flammeus) and black-chested buzzard-eagle (Geranoaetus melanoleucus).9 Degus adjust their use of open and sheltered microhabitats in response to risk and thermal conditions.10
Foraging in groups can improve detection of predators in exposed places.11 Vegetation may provide concealment while also obstructing sightlines; vigilance therefore depends on the type and amount of cover, rather than simply increasing or decreasing whenever grass is present.12
Social behaviour
Groups and communication
Wild groups may contain several adult females and one or more males, with neighbouring groups using adjacent burrow systems. Membership can change as animals disappear, disperse or join other groups.13 Social instability in a particular study does not establish that natal-site fidelity, or philopatry, never occurs. Nor should a wild sex ratio be copied as a recommendation to create breeding groups in captivity.
Degus use a complex vocal repertoire. One study described fifteen call categories associated with contexts such as alarm, adult contact, aggression, juvenile distress and reproduction. Not every call’s meaning or function is fully established, so human-like interpretations such as announcing a “happy event” should be avoided.14
Non-vocal interactions include mutual grooming, close investigation of the face or mouth, chasing, mounting outside mating and resting in physical contact. Chasing can occur in different contexts, including play and conflict. Social networks and interaction patterns also vary with reproductive state, including lactation.15
Diet and foraging
Degus are herbivorous and largely folivorous, eating leaves and stems together with roots, seeds, bark and some fruit. They can climb shrubs to obtain food. Occasional insect material has also been reported, but this does not make animal protein a routine dietary requirement. Foraging takes them away from burrow entrances into areas where food quality, cover and predator risk must be balanced.
Seasonal resource use and habitat disturbance affect population patterns; a study in La Campana National Park also discussed palm fruit as a nutritional resource.16 Seed handling can contribute to dispersal as well as seed predation, with context-dependent effects on vegetation. See the degu’s natural diet in Chile for a more detailed account.
Reproduction and development
Seasonal reproduction and gestation
Reproduction is affected by photoperiod and ecological conditions; it cannot be reduced to the circadian rhythm alone. Degus are also studied more broadly in chronobiology and translational medicine.17 Field studies commonly describe a main annual breeding season, with a second reproductive episode in some populations or favourable conditions. Litter size varies, with around five young often reported.24
Historical observations, including those associated with Thomas Bridges, should not be turned into a universal two-litters-per-year rule. Fulk’s field study was published in 1976 and reported substantial reproductive activity around September near Santiago. July and August are winter in the Southern Hemisphere, not summer. Gestation lasts about ninety days—long compared with mice and rats, but not the longest among all rodents. For comparison, a cheetah’s gestation is also approximately three months.918
Care of the young
Females may share a nest and nurse young other than their own. A study found no discrimination in nursing under its test conditions,19 while separate olfactory experiments showed that mothers can distinguish the odours of their own young from those of a co-nesting partner. These findings address different behaviours and are not contradictory.20
Fathers also participate in contact and social interactions with young; reported play and dominance behaviours depend on the setting.21 The study titled No infanticide found no infanticide under its particular conditions, but does not prove that it never occurs in the wild or captivity.22 Historical observations of shared burrows with other rodents likewise do not justify assuming that any species can safely be housed together.7
Pups are born furred, with eyes open or opening, and can move within hours. Birth weights around 14 g are reported. They are more developed than newborn rats or mice but remain dependent on appropriate care and thermal conditions.1 Practical weaning ages vary; eight weeks is the approximate figure given in the original guide, while the dental-development study recommends a minimum of six weeks. Dental changes around day 72 concern functional occlusion, not a universal natural weaning age or the end of tooth growth.25 Sexual maturity varies widely, with historical reports ranging from roughly two to nine months; maturity is not a recommendation to breed a young animal.
Sources
Woods, C. A., & Boraker, D. K. (1975). Octodon degus. Mammalian Species, 67, 1–5. https://doi.org/10.2307/3503820
Hurley, M. J., et al. (2018). The long-lived Octodon degus as a rodent drug discovery model for Alzheimer’s and other age-related diseases. Pharmacology & Therapeutics, 188, 36–44. https://doi.org/10.1016/j.pharmthera.2018.03.001
Encyclopaedia Britannica (n.d.). Degu. https://www.britannica.com/animal/degu
Visticot, M.-E. C. (2002). Un nouvel animal de compagnie : l’octodon, Octodon degus. Veterinary doctoral thesis, École nationale vétérinaire d’Alfort. https://theses.vet-alfort.fr/telecharger.php?id=340
SAAVEDRA, BÁRBARA & SIMONETTI, JAVIER A (2003). Distribución holocénica de roedores octodóntidos en Chile central. Revista chilena de historia natural, 76(3), 383–389. https://scielo.conicyt.cl/scielo.php?script=sci_arttext&pid=S0716-078X2003000300004
TOKIMOTO, N. & OKANOYA, K. (2004). Spontaneous construction of “Chinese boxes” by Degus (Octodon degu): A rudiment of recursive intelligence?1. Japanese Psychological Research, 46(3), 255-261. https://doi.org/10.1111/j.1468-5584.2004.00257.x
BENNETT, E. T. (1839). On the Genus Octodon, and on its Relations with Ctenomys, Blainv., and Poephagomys, F. Cuv.: including a Description of a New Species of Ctenomys. The Transactions of the Zoological Society of London, 2(1), 75-86. https://doi.org/10.1111/j.1469-7998.1839.tb00010.x
Meserve, P. L. & Gutiérrez, J. R. & Jaksic, F. M. (1993). Effects of vertebrate predation on a caviomorph rodent, the degu (Octodon degus), in a semiarid thorn scrub community in Chile. Oecologia, 94(2), 153–158. https://link.springer.com/article/10.1007/BF00341311
Fulk, G. W. (1976). Notes on the activity, reproduction, and social behavior of Octodon degus. Journal of Mammalogy, 57(3), 495–505. https://doi.org/10.2307/1379298
Lagos, V. O., Bozinovic, F., & Contreras, L. C. (1995). Microhabitat use by a small diurnal rodent (Octodon degus) in a semiarid environment: Thermoregulatory constraints or predation risk?. Journal of Mammalogy, 76(3), 900–905. https://doi.org/10.2307/1382759
Ebensperger, L. A. & Wallem, P. K. (2002). Grouping increases the ability of the social rodent,
Octodon degus
, to detect predators when using exposed microhabitats. Oikos, 98(3), 491-497. https://doi.org/10.1034/j.1600-0706.2002.980313.x
Ebensperger, L. A. & Hurtado, M. J. (2005). On the Relationship between Herbaceous Cover and Vigilance Activity of Degus (Octodon degus). Ethology, 111(6), 593-608. https://doi.org/10.1111/j.1439-0310.2005.01084.x
Ebensperger, L. A., et al. (2009). Instability Rules Social Groups in the Communal Breeder RodentOctodon degus. Ethology, 115(6), 540-554. https://doi.org/10.1111/j.1439-0310.2009.01635.x
Long, C. V. (2007). Vocalisations of the degu Octodon degus, a social caviomorph rodent. Bioacoustics, 16(3), 223–244. https://doi.org/10.1080/09524622.2007.9753579
Wey, T. W., et al. (2013). Reproductive correlates of social network variation in plurally breeding degus (Octodon degus). Anim Behav, 85(6), 1407-1414. https://doi.org/10.1016/j.anbehav.2013.03.035
Zunino, S., & Saiz, F. (1991). Estructura y densidad poblacional de Octodon degus Mol.. Studies on Neotropical Fauna and Environment, 26(3), 143–148. https://doi.org/10.1080/01650529109360846
Frontiers (n.d.). Octodon degus: An animal model that benefits translational medicine. Research Topic collection. https://www.frontiersin.org/research-topics/12583/octodon-degus-an-animal-model-that-benefits-translational-medicine
San Diego Zoo Wildlife Alliance (n.d.). Cheetah. https://animals.sandiegozoo.org/animals/cheetah
Ebensperger, L. A., Hurtado, M. J. & Valdivia, I. (2006). Lactating Females Do Not Discriminate Between Their Own Young and Unrelated Pups in the Communally Breeding Rodent, Octodon degus. Ethology, 112(9), 921-929. https://doi.org/10.1111/j.1439-0310.2006.01251.x
Jesseau, S. A., Holmes, W. G., & Lee, T. M. (2008). Mother–offspring recognition in communally nesting degus, Octodon degus. Animal Behaviour, 75(2), 573–582. https://doi.org/10.1016/j.anbehav.2007.06.015
Wilson, S. C. (1982). Contact‐promoting behavior, social development, and relationship with parents in sibling juvenile degus (Octodon Degus). Developmental Psychobiology, 15(3), 257-268. https://doi.org/10.1002/dev.420150309
Ebensperger, L. A. (2001). No infanticide in the hystricognath rodent, Octodon degus: does ecology play a role?. acta ethologica, 3(2), 89–93. https://link.springer.com/article/10.1007/s102110000032
CONAF (2024). Después de 65 años encuentran al degú en la Reserva Nacional Isla Mocha. https://www.conaf.cl/despues-de-65-anos-encuentran-al-degu-en-la-reserva-nacional-isla-mocha/
Meserve, P. L., Martin, R. E., & Rodríguez, J. (1984). Comparative ecology of the caviomorph rodent Octodon degus in two Chilean Mediterranean-type communities. Revista Chilena de Historia Natural, 57, 79–89. https://rchn.biologiachile.cl/pdfs/1984/1/Meserve_et_al_1984.pdf
Jekl, V., et al. (2011). Dental eruption chronology in degus (Octodon degus). Journal of Veterinary Dentistry, 28(1), 16–20. https://doi.org/10.1177/089875641102800103