The diet of wild degus varies with season, habitat and available resources. They are herbivorous and largely folivorous, consuming leaves and stems as well as seeds, roots, bark and some fruit. In captivity, a suitable diet helps reduce nutritional risk, but cannot prevent every illness. Commercial foods must be assessed by their composition: a degu label does not guarantee a match to the species’ needs.
Feeding in the wild
A selective forager
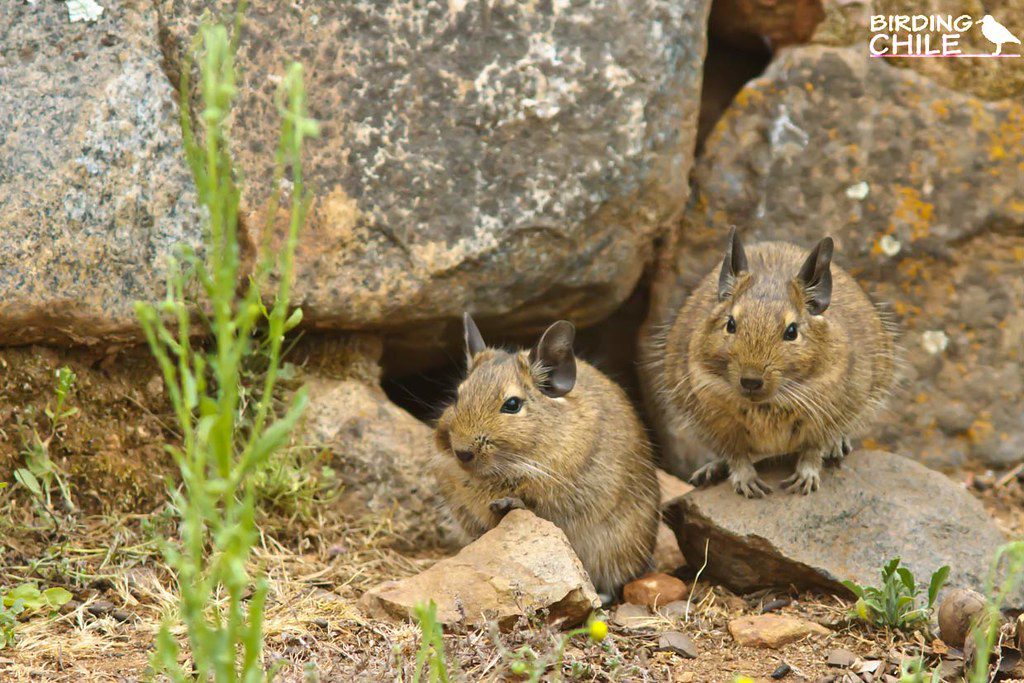
In their natural habitat, degus spend considerable time searching for food, eating some immediately and storing some for later. They gather much of their food at ground level, but also climb shrubs to reach leaves, fruit and bark. When food is abundant, they may concentrate their activity near the burrow.
Older natural-history accounts report feeding on plants such as Cestrum parqui and Vachellia caven, formerly referred to as Acacia caven or Mimosa cavenia.1 Other plants mentioned in dietary and habitat accounts include Erodium cicutarium, Proustia cuneifolia, Atriplex repanda, Porlieria chilensis, Colliguaya odorifera, Kageneckia oblonga, Quillaja saponaria, Proustia pungens, Lithraea caustica, Chenopodium petiolare and Nassella pubiflora.2 Hawthorn fruit and thistle seeds also appear in the original account; its identification of thistles as Ageratum was unsupported. These descriptive wild records are not a list of plants recommended for captive feeding.
Seasonal variation
At a central Chilean study site, grasses and other herbaceous plants were important, while acacia tissues were eaten during the dry months of January–April. Moisture in shrub tissues may contribute to their seasonal value. The original dietary analysis reports seed contributions of 63.1% in November and 29.3–60.0% during December–April. These figures describe particular samples and seasons, rather than a fixed requirement. Shrub seeds become available after flowering, while seeds of annual plants remain on the ground after vegetation has dried. Such food can be important for juveniles.3
Food selection and storage
Degus often select young shoots over older leaves, potentially benefiting from their water and protein content. When alternatives are available, they may favour foods with more protein and less fibre, although their overall ecology remains that of a herbivorous rodent.4 Food quality and nitrogen availability help explain why abundant vegetation may constitute a nutritional “green desert”: much of what is present may not be preferred or sufficiently nutritious. This does not mean that degus create a desert by eating selected plants.5
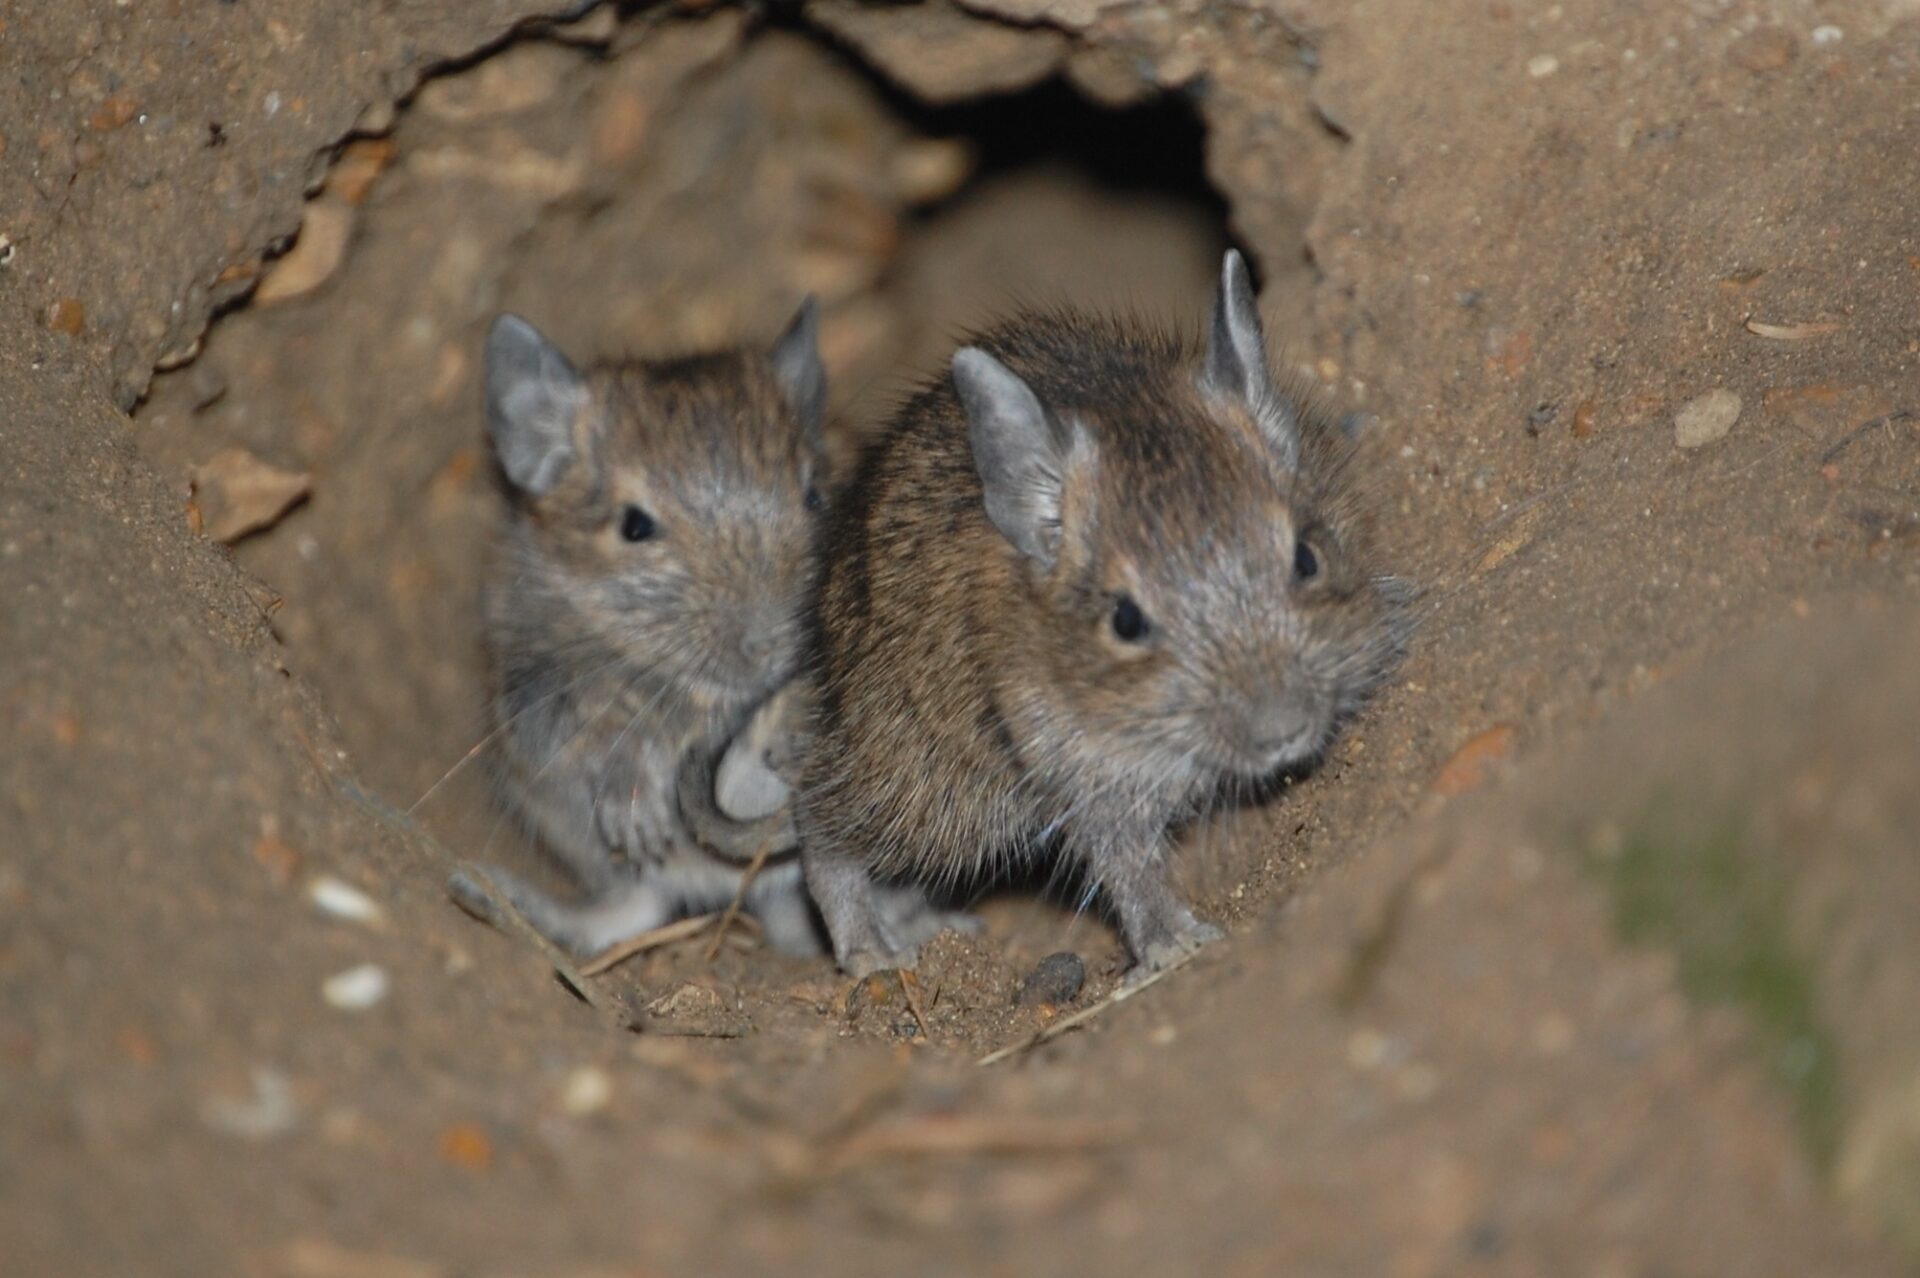
Food-storage behaviour also differs between populations. In a study comparing animals from high- and low-altitude sites, high-altitude degus used both central larder stores and scattered caches, whereas the low-altitude animals used scatter hoarding. High-altitude animals were smaller, but seed consumption adjusted for body mass did not differ significantly. These laboratory comparisons should not be simplified to a universal rule that all mountain degus eat less.6
Ecological roles
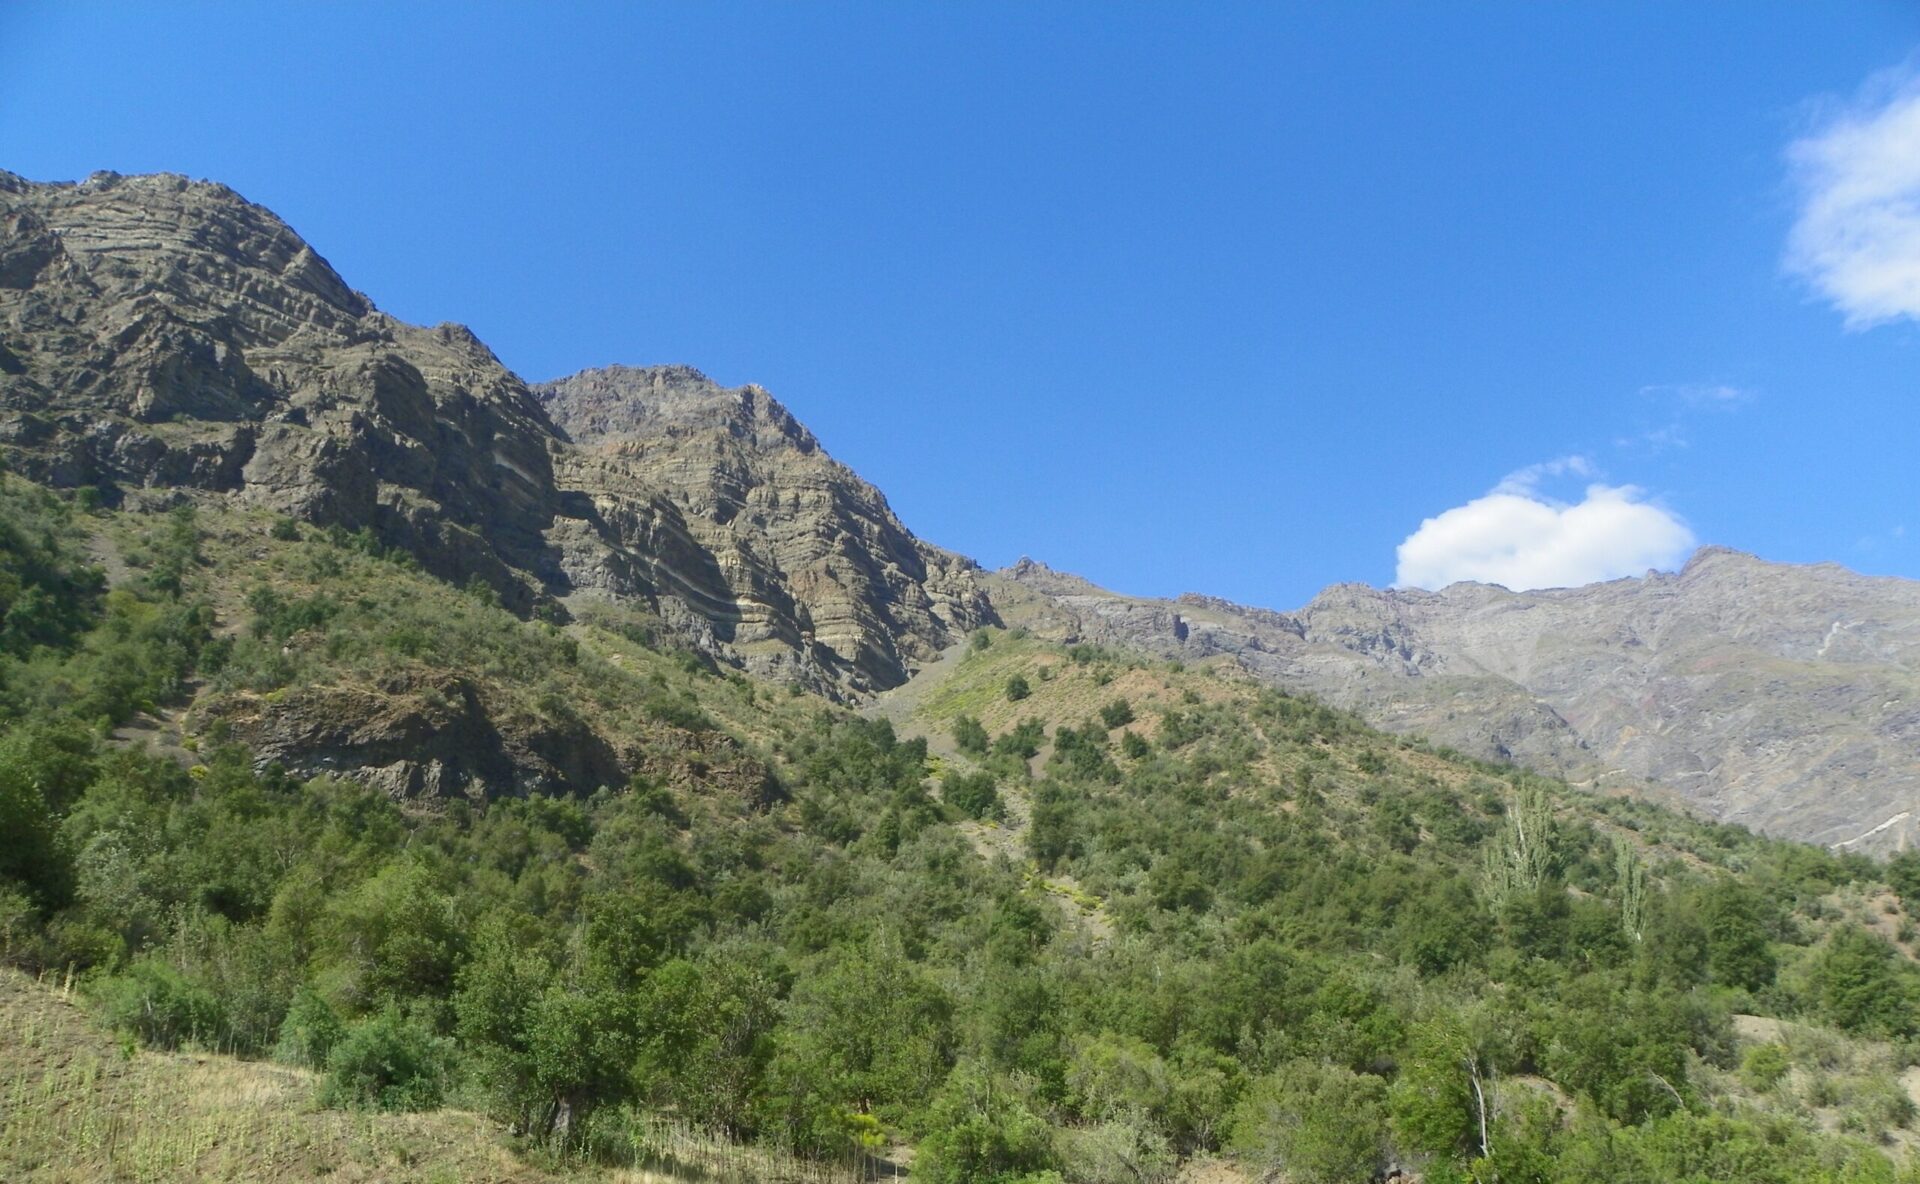
Degus occupy a range of Chilean environments, including matorral, plains, mountain areas and some wooded or modified habitats. They are common caviomorph rodents in several Mediterranean-type communities. Chile does have native large herbivores; the ecological importance of degus does not depend on their absence. Introduced livestock, including goats, add different pressures.
Feeding, movement, caching and burrowing all influence the surrounding vegetation and soil. Their effects depend on context, rather than being uniformly beneficial or harmful.
Vegetation and seed dispersal
Leaves and other vegetative tissues can form a large fraction of the diet—figures around 60% are reported in some contexts—but vary greatly by site and season. Grazing near burrows changes local cover and may favour some plants over others. Seeds can be eaten, cached, moved or left uneaten. Research shows that rodents may act as both seed predators and dispersers, with outcomes depending on food availability and other conditions.7 The earlier figure of a general 12 m dispersal radius should not be treated as a universal movement distance.
Repeatedly used paths, disturbed soil and accumulations of twigs or litter around burrows may also affect where plants establish.
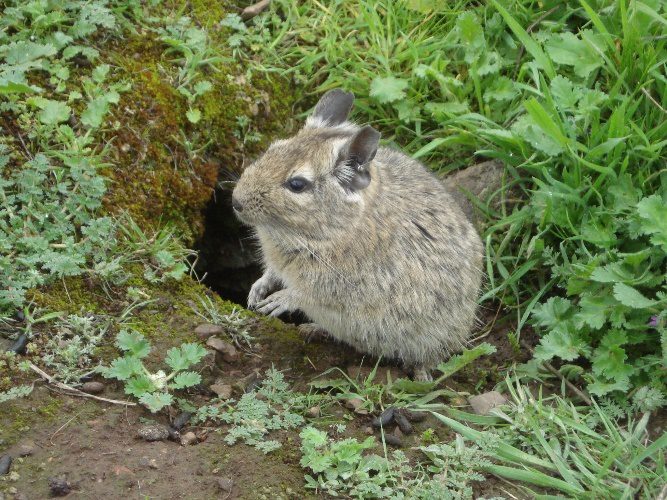
Context-dependent effects on matorral
Feeding on young shoots can limit individual shrubs, while seed movement and soil disturbance may aid other plants. Habitat selection depends on cover and other local conditions, and does not imply either preference for one shrub everywhere or complete ecological neutrality.8
In arid habitats, perennial plants become particularly important. Droppings contribute nutrients to soil, and annual plants such as Moscharia pinnatifida may benefit from locally enriched conditions. Degus can process fibrous food through hindgut fermentation, but this does not mean that they generally avoid annual vegetation or only transport its seeds. Experimental work shows that the effects of small mammals on plants depend on interactions with predators and environmental conditions.9
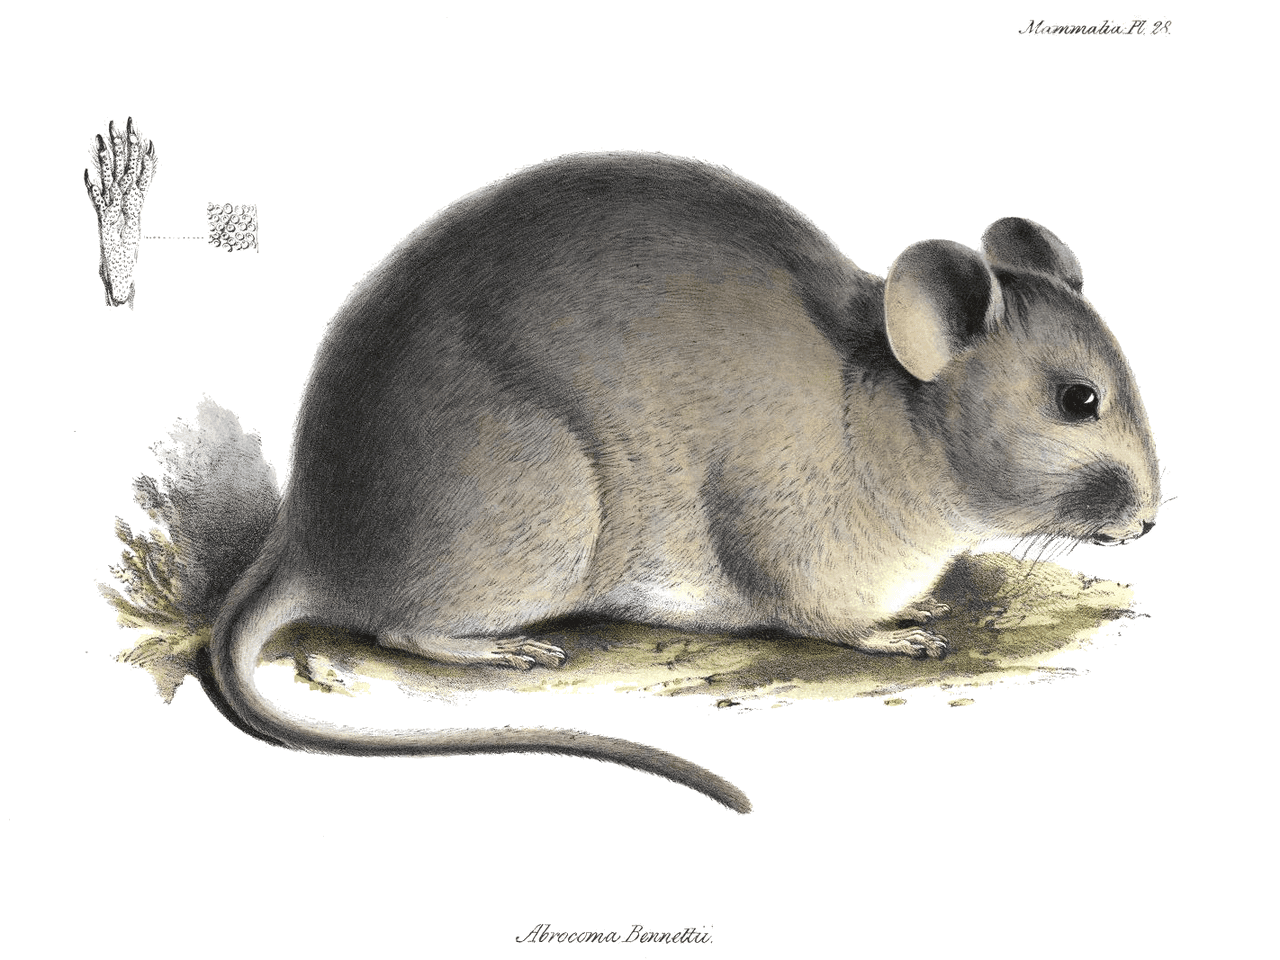
Degus share habitats with other rodents, including Bennett’s chinchilla rat (Abrocoma bennettii), whose diet overlaps in some respects.2 Other associated species include the olive grass mouse, historically called Akodon olivaceus and now Abrothrix olivacea, Abrothrix longipilis and Phyllotis darwini. Coexistence and dietary differences do not, by themselves, prove that competition never occurs.
Habitat differences and human influence
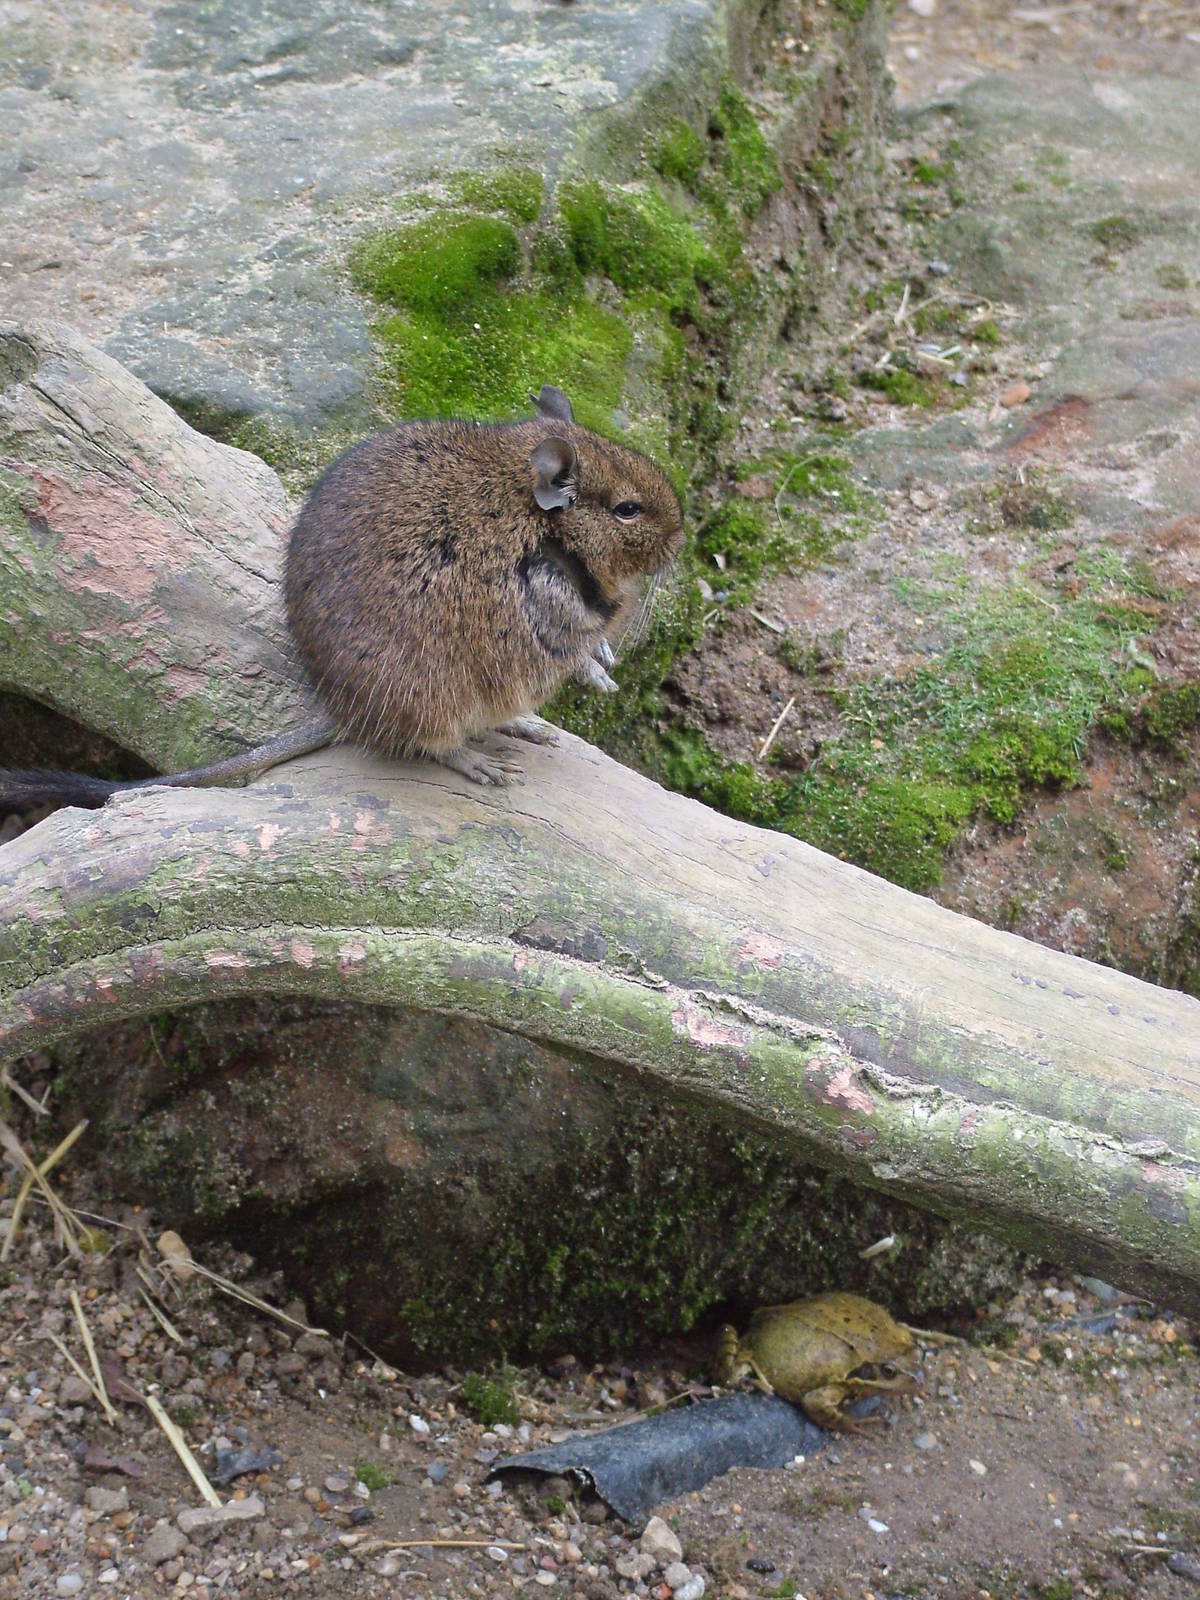
Comparisons at Fray Jorge and La Dehesa illustrate how strongly local conditions affect diet. The original account reports spring shrub cover of 59.6% and herbaceous cover of 21.7% at the Fray Jorge site. Herbaceous foliage was less prominent in the diet except during September and November, when values of 45.8–73.3% were reported; grass seeds did not exceed 6.9%. Shrub foliage contributed approximately 44.6%, compared with 18.7% at La Dehesa. Evergreen shrubs such as Chenopodium petiolare may supply moisture during dry months. These are study-site observations, not species-wide nutritional prescriptions.2
Degus generally use habitats with shelter such as shrubs or rocks, but also occur in degraded grasslands and marginal agricultural land. Overgrazing, burning and removal of fuelwood can favour shrubs including Vachellia caven, Lithraea caustica, Puya and Baccharis. Their occurrence in these disturbed landscapes may therefore be a consequence of habitat change, rather than its original cause. Long-term work at Bosque Fray Jorge also demonstrates the importance of interactions among climate, plants, small mammals and predators.10
Protecting the habitat
Introduced herbivores such as hares and goats, alien plants, urban expansion and pollution can alter these ecosystems and affect degus. Protecting and appropriately managing natural habitats helps conserve both the animals and the ecological relationships in which they participate.
Sources
Woods, C. A., & Boraker, D. K. (1975). Octodon degus. Mammalian Species, 67, 1–5. https://doi.org/10.2307/3503820
Meserve, P. L., Martin, R. E., & Rodríguez, J. (1984). Comparative ecology of the caviomorph rodent Octodon degus in two Chilean Mediterranean-type communities. Revista Chilena de Historia Natural, 57, 79–89. https://rchn.biologiachile.cl/pdfs/1984/1/Meserve_et_al_1984.pdf
Meserve, P. L., Martin, R. E. & Jaime, R. M. (1983). Feeding Ecology of Two Chilean Caviomorphs in a Central Mediterranean Savanna. Journal of Mammalogy, 64(2), 322-325. https://doi.org/10.2307/1380568
Edwards, M. S. (2009). Nutrition and Behavior of Degus (Octodon degus). Veterinary Clinics of North America: Exotic Animal Practice, 12(2), 237-253. https://doi.org/10.1016/j.cvex.2009.01.003
Gutiérrez, J. R. & Bozinovic, F. (1998). Diet selection in captivity by a generalist herbivorous rodent (Octodon degus) from the Chilean coastal desert. Journal of Arid Environments, 39(4), 601-607. https://doi.org/10.1006/jare.1998.0412
Quispe, R., et al. (2009). Inter‐Population Variation in Hoarding Behaviour in Degus,Octodon degus. Ethology, 115(5), 465-474. https://doi.org/10.1111/j.1439-0310.2009.01621.x
Loayza, A. P., Luna, C. A. & Calviño-Cancela, M. (2020). Predators and dispersers: Context-dependent outcomes of the interactions between rodents and a megafaunal fruit plant. Scientific Reports, 10(1), 6106. https://doi.org/10.1038/s41598-020-62704-6
Simonetti, Javier A. & Montenegro, Gloria (1981). Food preferences by Octodon degus (Rodentia caviomorpha): Their role in the chilean matorral composition. Oecologia, 51(2), 189–190. https://link.springer.com/article/10.1007/BF00540599
Gutiérrez, J. R., et al. (1997). Effects of small mammals and vertebrate predators on vegetation in the Chilean semiarid zone. Oecologia, 109(3), 398-406. https://doi.org/10.1007/s004420050099
GUTIÉRREZ, J. R., et al. (2010). Long-term research in Bosque Fray Jorge National Park: Twenty years studying the role of biotic and abiotic factors in a Chilean semiarid scrubland. Revista chilena de historia natural, 83(1). https://doi.org/10.4067/s0716-078×2010000100005